Meta Analysis
Analysis of Wild Resource Decline and Artificial Germplasm Restoration Pathways of Paris spp. 

 Author Correspondence author
Medicinal Plant Research, 2026, Vol. 16, No. 4
Received: 20 Jun., 2026 Accepted: 08 Aug., 2026 Published: 23 Aug., 2026
Paris spp. are important medicinal plant resources in China, and their rhizomes are rich in bioactive compounds, particularly steroidal saponins, which possess high medicinal value and considerable potential for industrial utilization. However, long-term dependence on wild harvesting, habitat degradation, and limited natural regeneration capacity have resulted in continuous declines of wild Paris resources, increasing the risk of losing valuable germplasm and making it difficult to meet the sustainable development needs of the traditional Chinese medicine industry. This study investigates the causes of wild resource decline and the pathways for artificial germplasm restoration of Paris spp. This article analyzes population dynamics, and impacts of excessive harvesting and ecological changes on resource stability. Furthermore, the major constraints in artificial germplasm development are summarized, including high dependence on wild germplasm sources, long propagation cycles, insufficient rapid propagation systems, and incomplete genetic background and quality evaluation frameworks. To address these challenges, this study proposes a restoration strategy based on wild germplasm conservation and elite germplasm selection, supported by efficient propagation technologies, understory ecological cultivation, and standardized production systems. The potential applications of molecular markers, genomics-assisted breeding, and long-term resource management strategies in Paris germplasm innovation are also discussed. Future efforts should focus on wild resource conservation, core germplasm construction, precise evaluation of elite materials, and ecological adaptation-based cultivation to promote the transition of Paris resource utilization from wild collection-dependent exploitation toward artificial germplasm-driven and ecologically sustainable production systems. This review proposes theoretical references for genetic resource conservation, stable medicinal material supply, and sustainable industrial development of Paris spp.
1 Introduction
Paris spp. are a group of medicinally important perennial herbs with long-standing use in Asian traditional medicine and substantial contemporary value for the pharmaceutical industry. The genus has been used in China for more than 2 000 years, and several Paris taxa, especially P. polyphylla, P. polyphylla var. yunnanensis, and P. polyphylla var. chinensis, are widely employed in ethnomedicine and formal medicinal systems for treating trauma, bleeding, inflammation, swelling, skin disorders, and related conditions (Jiang et al., 2022; Ye et al., 2025). Modern phytochemical and pharmacological studies show that Paris species are rich in bioactive secondary metabolites, especially steroidal saponins, which account for more than 80% of identified active compounds and are regarded as the principal medicinal constituents and chemotaxonomic markers of the genus (Ding et al., 2021; Rawat et al., 2023; Zhang et al., 2025). Since 1960, more than 320~330 compounds have been isolated from Paris plants, including steroidal saponins, flavonoids, phytosterols, triterpenes, polysaccharides, and related constituents, reflecting both chemical richness and broad development potential (Thapa et al., 2022). Representative steroidal saponins such as polyphyllins and Paris saponins exhibit anticancer, hemostatic, anti-inflammatory, antimicrobial, antiviral, immunomodulatory, and other activities, and recent compound-level studies continue to identify new molecules with notable cytotoxic or anti-inflammatory effects (Thakur et al., 2023). This medicinal importance has driven intense utilization of rhizomes as the source material for traditional remedies and for more than 100 proprietary Chinese medicines, making Paris spp. both biologically valuable and economically strategic (Kunwar et al., 2020).
However, the same high medicinal and commercial value that has promoted the use of Paris spp. has also accelerated the depletion of wild resources. Before the 2000s, Paris species were not cultivated in plantations, and the pharmaceutical industry relied primarily on Rhizoma Paridis collected from wild populations; with annual raw-material consumption estimated at about 3 000 000 kg, overharvesting has caused dramatic declines in natural populations. Multiple studies identify overexploitation, illegal collection, habitat degradation, habitat fragmentation, logging, farming, trampling, and weak management as key drivers of decline, and several reviews now describe P. polyphylla as vulnerable, endangered, or rare and threatened in different regional and conservation contexts (Thapa et al., 2022; Thakur et al., 2023). Field evidence from the Indian Himalayan Region recorded very low population densities of only 0.42~1.48 individuals/m2 and emphasized that unsustainable extraction, poor natural regeneration, and rhizome-focused harvesting place wild populations at risk of local extinction. Similar patterns are reported from Nepal, where accelerating demand has promoted unsustainable legal and illegal harvest, premature collection, and habitat degradation, while trade pressure continues across broad distribution areas (Kunwar et al., 2020). Recent cultivation-oriented work further underscores the severity of the supply crisis, noting that approximately 80% of wild resources are exploited annually and that, in Yunnan alone, demand exceeds 1 000 tons while annual wild production is less than 100 tons (Zhang et al., 2025). Because Paris species also grow slowly, regenerate inefficiently, and often depend on harvested rhizomes for both medicinal use and vegetative persistence, wild-resource decline has become a coupled ecological and industrial problem (Wang et al., 2021).
Under these conditions, artificial germplasm restoration has become essential for both conservation and sustainable utilization of Paris spp. Conventional propagation remains constrained by slow seed germination, secondary dormancy, long juvenile growth, low multiplication rates, and disease or rot associated with rhizome cutting, while interspecific hybridization can also compromise the uniformity of medicinal raw materials and complicate seed-based breeding. These constraints explain why traditional breeding and propagation have not kept pace with rising herbal-drug demand and why researchers increasingly emphasize ex situ conservation, clonal multiplication, and tissue-culture-based restoration pathways (Thapa et al., 2022). Encouragingly, several studies have demonstrated feasible artificial propagation routes. Direct somatic embryogenesis has achieved successful regeneration with high germination and ploidy stability in regenerated plants. In vitro propagation using optimized plant growth regulators has produced strong shoot induction and 94.4% greenhouse establishment (Puwein and Thomas, 2022). GA3 treatment can rapidly break dormancy and induce polyapical shoots at 100%, offering a more efficient rhizome propagation strategy. Somatic embryogenesis-based clonal propagation can also generate homogeneous elite materials, support cryopreservation-compatible conservation, and shorten plantlet production by 12~15 months while maintaining favorable biomass and saponin traits (Wang et al., 2023). In parallel, emerging work on seed dormancy regulation indicates that improving reproductive efficiency remains a central scientific challenge for large-scale restoration.
Accordingly, research on the decline of wild Paris resources and the pathways for artificial germplasm restoration has both theoretical and practical significance. At the scientific level, the taxonomic complexity of the genus, disputed species boundaries based on morphology, and demand for robust phylogenetic markers indicate that conservation must be linked with accurate germplasm identification and genetic-resource management. At the applied level, restoration research should clarify patterns of wild-resource depletion, identify the biological bottlenecks limiting natural and artificial regeneration, screen elite germplasm with stable medicinal quality, and integrate in situ protection, ex situ conservation, standardized cultivation, and traceable supply systems. It should also connect germplasm restoration with quality formation, since saponin accumulation varies with developmental stage and growth duration, making the relationship between propagation strategy, growth years, and medicinal quality especially important for sustainable production. More broadly, effective restoration can reduce harvesting pressure on wild populations, preserve genetic diversity, stabilize raw-material supply, support rural cultivation economies, and improve the long-term sustainability of biodiversity use under intensifying market demand. For these reasons, analyzing wild resource decline and constructing practical artificial germplasm restoration pathways for Paris spp. is a necessary foundation for reconciling medicinal use, industrial development, and species conservation.
2 Current Status and Main Factors Driving the Decline of Wild Paris spp. Resources
2.1 Distribution characteristics and population changes of wild resources
Paris spp. are distributed mainly in temperate and subtropical mountain systems of Eurasia, with clear diversity centers in Southwest China and the Himalayan region. The genus has been described as a small but taxonomically complex understory herb group concentrated in East Asia, with the Yunnan-Guizhou Plateau recognized as a major center of diversity, while P. polyphylla is reported across Bhutan, China, India, Laos, Myanmar, Nepal, Thailand, and Vietnam (Ding et al., 2021). Within this broad range, wild populations show strong geographic structuring and uneven local occurrence. In Nepal, field surveys recorded the species in 51 districts, while use and trade records were concentrated in fewer districts, indicating spatial heterogeneity in occurrence and exploitation intensity (Kunwar et al., 2020). Genetic and phylogeographic studies further show obvious geographic structure in wild populations of P. polyphylla var. yunnanensis, with Guizhou and western Yunnan identified as important conservation areas because they retain distinctive wild lineages and higher diversity (Huang et al., 2019; Zhao et al., 2021).
Despite this relatively wide distribution, most studies describe wild resources as sparse, fragmented, and declining. Field surveys in Arunachal Pradesh reported densities ranging from 0.42 to 1.48 individuals/m2 in one study and 2.48 to 8.2 individuals/m2 in another, showing that local populations can persist but are often thin and highly site-dependent (Kalita et al., 2026). In Sikkim, density ranged from 0.45 to 3.89 plants/m2, and in Manipur from 1.3 to 2.4 individuals/m2, again indicating low to moderate abundance with substantial variation among habitats (Lepcha et al., 2019; Singh et al., 2026). Nepalese ecological work reported an average density of only 1.78 individuals/m2, while recent reviews note that many contemporary wild populations now occur as small isolated groups, with larger populations mostly restricted to remote areas or protected sites (Ye et al., 2025). Across regions, the consensus is that wild Paris resources are undergoing continuous decline under combined pressure from overexploitation, illegal collection, and habitat degradation, and several papers explicitly describe the taxa as vulnerable, endangered, or at risk of extinction (Thakur et al., 2023).
2.2 Effects of excessive harvesting on wild population regeneration
Excessive harvesting is the most consistently identified direct driver of wild Paris decline because medicinal use depends primarily on rhizomes, the same organs that support perennial survival and vegetative regeneration. Reviews and field studies agree that demand has risen rapidly in recent decades, stimulating both legal and illegal trade and intensifying extraction across China, Nepal, India, and neighboring range states (Cunningham et al., 2018; Kunwar et al., 2020). Price escalation has reinforced this pressure: one review documented a roughly 400-fold rise in rhizome prices in China since the 1980s, while more recent work notes that soaring prices since 2013 have encouraged large-scale farmer collection from wild stands. Because human activity is repeatedly identified as the primary factor affecting population size, commercially valuable populations near settlements or trade routes appear especially vulnerable to depletion (Singh et al., 2026).
The biological consequences of overharvesting are severe because Paris regenerates slowly and reproduces inefficiently under disturbance. Several studies state that the rhizome is the principal mode of regeneration in the field, while seed-based recruitment is constrained by low viability, poor germination, and long dormancy. Harvesting before seed maturation is singled out as especially damaging because it reduces seed formation and germination and removes plants before recruitment can occur (Thapa et al., 2022). Competitive and unscientific collection practices often remove the whole underground portion without leaving propagative fragments, directly interrupting vegetative recovery and accelerating population collapse. This harvesting pressure interacts with intrinsic life-history limits, including slow growth, delayed reproductive maturity, many non-flowering individuals, and lengthy breeding cycles, so wild populations recover far more slowly than they are being depleted (Ye et al., 2025).
2.3 Habitat alteration and ecological adaptation stress
Wild Paris populations are also highly sensitive to habitat alteration because the plants occupy relatively narrow understory niches. Ecological studies consistently place P. polyphylla in shady, moist, relatively undisturbed forest habitats, commonly under canopy cover greater than 80%, in humus-rich, well-drained soils, and often on slopes or streamside microsites (Singh et al., 2026). Distribution modeling reinforces that this niche is environmentally constrained: precipitation, elevation, slope, vegetation type, and temperature range were all identified as important predictors of suitable habitat in regional models from Sikkim, Uttarakhand, and China (Tariq et al., 2021; Wang et al., 2026). Disturbed habitats repeatedly show poorer agreement with predicted suitable occurrence, implying that even climatically suitable areas may fail to support stable populations once human disturbance alters forest structure (Lepcha et al., 2019).
Habitat degradation therefore acts not only by reducing area, but by imposing ecological stress that suppresses growth and reproduction. Forest loss, fragmentation, logging, agricultural expansion, slash-and-burn cultivation, fire, landslides, grazing, trampling, and urbanization are all reported as pressures that thin populations and degrade understory conditions (Singh et al., 2026). Experimental and field evidence indicates that the species has poor adaptability to altered environments and reduced reproductive vigor under changed climatic or habitat conditions, while less than 50% shade significantly lowers seed productivity and waterlogging can be lethal. Metapopulation modeling from Sikkim further shows that disturbance and forest fragmentation substantially worsen long-term persistence, increasing extinction risk under disturbed scenarios and supporting the priority of protecting reproductive individuals in undisturbed forest matrices (Lyngdoh et al., 2018). Overall, the decline of wild Paris spp. reflects the interaction of commercial overexploitation with narrow habitat requirements and weak natural regeneration, making integrated in situ protection, cultivation, and habitat restoration necessary for long-term conservation (Thakur et al., 2023).
3 Current Status and Key Constraints of Artificial Germplasm Development in Paris spp.
3.1 Dependence on wild germplasm sources and insufficient foundations for artificial propagation
Artificial germplasm development in Paris spp. remains strongly dependent on wild resources, because domestication has started late and cultivated materials are still closely tied to wild-collected source populations. Several studies note that wild P. polyphylla has been excessively harvested and pushed toward endangerment, while cultivation has been promoted mainly as a compensatory response to the collapse of natural supplies rather than as a long-established breeding system (Puwein and Thomas, 2019; Tang et al., 2022). This weak domestication history is reflected genetically: cultivated and wild populations show little differentiation in some marker studies, with only 1.35% variation reported between 15 wild and 17 cultivated populations, indicating that cultivated stocks still largely derive from recently introduced and mixed wild origins rather than from stabilized breeding lines (Huang et al., 2019). At the same time, artificial cultivation has become essential because wild resources are now rare, and some cultivation-population studies were conducted precisely because representative planting areas already depended on scarce wild germplasm collected earlier from multiple origins (Gao et al., 2022).
The second constraint is that the biological basis for large-scale artificial propagation remains weak. Paris spp. show long growth cycles of about 7~10 years, extremely long dormancy release, and low reproductive efficiency, which together create a persistent bottleneck for seedling production and industrial planting (Wang et al., 2023). Seeds require more than 18 months to break dormancy in some studies, only about 40% germinate under natural conditions, and dormancy is described as morphophysiological or “double dormancy,” which makes routine nursery establishment slow and unreliable (Tang et al., 2022). Even where artificial treatment improves germination, the gains remain limited: one seed-dormancy study achieved a 40% germination rate after combined cold storage, temperature fluctuation, infrared treatment, and chemical soaking, underscoring that the propagation foundation is still technically demanding rather than straightforward. Reviews therefore conclude that conventional breeding and propagation cannot keep pace with medicinal demand, and that advanced biotechnological approaches in Paris remain comparatively rare or insufficiently developed (Figure 1) (Rawat et al., 2023).
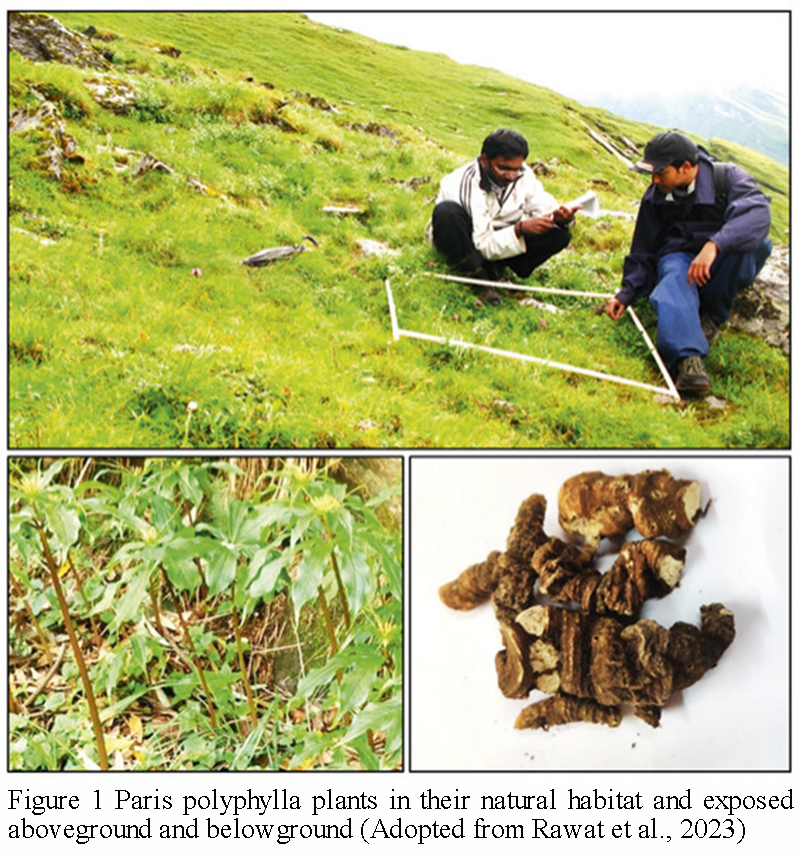 Figure 1 Paris polyphylla plants in their natural habitat and exposed aboveground and belowground (Adopted from Rawat et al., 2023) |
3.2 Limitations of Paris spp. propagation technologies
Current propagation technologies for Paris spp. have made clear progress, but each major route still carries practical limitations. Traditional rhizome cutting is widely used because the species grows slowly and clonal propagation can bypass seed dormancy, yet the method has low multiplication efficiency because axillary meristems are limited, and cutting can sharply reduce net rhizome yield (Wang et al., 2021). Rhizome injury also creates phytosanitary problems: cut segments are susceptible to insects, disease, and rotting, causing substantial yield losses during multiplication (Wang et al., 2023). Even when rhizome splitting works, propagation rates are variable rather than uniformly high. In one three-year study, sprouted shoot buds averaged 49.33% from cut rhizomes and 75% from group rhizome fragmentation, which is useful for conservation but still indicates incomplete and method-dependent conversion efficiency. Other patented or nursery-based methods improve latent-bud induction or avoid direct rhizome damage, but these are still technique-specific optimizations rather than evidence of a universally standardized propagation system.
In vitro propagation and hormone-based regulation offer promising alternatives, but they also show that successful multiplication depends on highly specific developmental stages, explant types, and culture conditions. Tissue culture protocols have reported strong outcomes, including 80% shoot response and 94.4% greenhouse establishment under optimized BAP and NAA conditions, while other systems achieved bud germination within 6~8 days, multiplication factors above 5, rooting rates above 90%, and transplant survival above 90% (Puwein and Thomas, 2022). Somatic embryogenesis can further increase scale, producing an average of 63 somatic embryos per gram of callus in six weeks and shortening plantlet production by 12~15 months (Wang et al., 2023). However, these gains depend on precise regulation of medium composition, photoperiod, sucrose concentration, temperature, plant growth regulators, and rhizome developmental stage, indicating that the technology remains sensitive and not yet simple for broad field deployment (Kumar et al., 2025). Hormone-based rhizome induction shows similar conditionality: GA3 can break dormancy within two weeks and induce polyapical shoots at 100%, with 7.2 apical shoots per treated rhizome, but this is still a controlled treatment protocol rather than a low-input routine practice for all germplasm types and planting settings (Wang et al., 2021).
3.3 Genetic background and quality evaluation deficiencies of artificial germplasm
A major constraint in artificial germplasm development is the incomplete understanding and control of genetic background. The genus has strong interspecific hybridization capacity, and unintended hybridization between P. polyphylla and related taxa can generate forms that are difficult to distinguish morphologically, which disrupts seed-based breeding and weakens the uniformity of medicinal raw materials. Marker studies also show that cultivated materials often carry high admixture and mixed ancestry. EST-SSR analysis found low differentiation among cultivated populations but high diversity among individuals, with populations likely derived from two ancestral groups and with evidence of cross-pollination among cultivars (Gao et al., 2022). AFLP results likewise showed that cultivated populations can have high variation, probably because they originated from mixed provenances, which means provenance screening is still urgently needed before artificial germplasm can be treated as genetically standardized breeding material (Huang et al., 2019).
Quality evaluation is similarly underdeveloped because medicinal value is not determined by survival alone, but by stable biomass and saponin accumulation across propagules, growth stages, and lineages. One recent study had to select elite wild accessions and then clone them as candidate cultivars on the basis of biomass production and polyphyllin content, showing that quality-assured artificial germplasm is still being built from screened wild founders rather than from mature breeding pools (Wang et al., 2023). Developmental-stage effects further complicate evaluation, because extraction yield, antioxidant activity, phenolics, flavonoids, and diosgenin content all change with plant age, and reproductive-stage rhizomes can differ substantially from juvenile or vegetative materials (Kumar et al., 2025). At the molecular level, researchers still emphasize that marker resources are limited, complete genomes are unavailable, EST resources are scarce, and the lack of marker information has constrained collection, conservation, and utilization of Paris germplasm (Gao et al., 2022). Although SSR, AFLP, SCoT, and SRAP studies now provide an emerging basis for diversity analysis and genetic improvement, these tools are still being established as foundational resources rather than functioning as a fully integrated quality-control system for artificial germplasm development (Zhao et al., 2020).
4 Key Technical Pathways for Artificial Germplasm Restoration of Paris spp.
4.1 Conservation of wild germplasm resources and selection of elite germplasm
Artificial germplasm restoration of Paris spp. should begin with the protection and systematic evaluation of wild germplasm, because wild populations remain the original reservoir of genetic diversity, adaptive traits, and medicinal-quality variation (Gao et al., 2022). Current evidence indicates that in situ conservation should remain the fundamental strategy even when ex situ cultivation and artificial propagation are expanding (Huang et al., 2019). Population genetic and phylogeographic studies show clear geographic structure in wild P. polyphylla var. yunnanensis, with Guizhou, western Yunnan, and parts of southern Sichuan retaining high conservation value and therefore deserving priority protection and restricted harvesting (Zhao et al., 2021). Wild populations in Guizhou appear especially important because they showed richer genetic diversity than those in Yunnan and were explicitly proposed as priority areas both for protection and for provenance selection. Broader regional work in Nepal and the Dabie Mountains similarly found substantial within-population variation and geographic clustering of germplasm, supporting region-based conservation sampling rather than random collection (Zhao et al., 2020; Oliya et al., 2023).
Elite germplasm selection should therefore combine ecological provenance, genetic diversity, and medicinal-quality screening instead of relying only on morphology or yield (Gao et al., 2022). This is especially necessary because cultivated populations often originate from mixed provenances and show admixture, gene flow, and weak domestication differentiation from wild sources, which can obscure genetic background and reduce breeding precision. Several studies now support using molecular markers such as AFLP, cpDNA haplotypes, SSR, EST-SSR, SCoT, and SRAP to define core germplasm, identify superior provenances, and guide conservation-oriented breeding (Zhao et al., 2020; Zhao et al., 2021). At the applied level, elite wild accessions have already been selected and clonally reproduced as candidate cultivars on the basis of biomass and saponin content, showing that restoration can move from passive conservation to targeted domestication when representative wild founders are first secured (Wang et al., 2023). Reasonable interventions in protected habitats, such as improving seed germination before sowing back into wild sites, may also strengthen renewal of effective wild populations and link conservation directly with germplasm recovery (Huang et al., 2019).
4.2 Establishment of efficient propagation technology systems
The second technical pathway is the establishment of efficient, scalable propagation systems that overcome the slow growth, long seed dormancy, and low multiplication efficiency of Paris spp. (Kumar et al., 2025). Conventional rhizome cutting remains useful, but its multiplication rate is limited by axillary meristem number and it can reduce net rhizome yield while increasing susceptibility to insects, disease, and rot (Wang et al., 2023). Improved rhizome-based techniques therefore focus on increasing bud activation without damaging the parent rhizome. Stratification-induced latent-bud propagation and related rapid seedling systems can raise propagation coefficient, preserve genetic stability, and produce robust field-surviving seedlings, while avoiding some of the losses associated with direct segment cutting. Hormone regulation offers another effective route: GA3 can break rhizome dormancy within two weeks and induce polyapical shoots at 100%, with about 7.2 apical shoots per treated rhizome, markedly improving clonal multiplication efficiency (Wang et al., 2021).
Tissue culture and somatic embryogenesis now appear to be the most promising high-efficiency restoration platform for large-scale artificial germplasm production (Thapa et al., 2022; Wang et al., 2023). Direct regeneration systems based on thin cell layer culture, mini-rhizome induction, and optimized hormone combinations have achieved 86.6% mini-rhizome formation, more than 95% acclimatization in greenhouse conditions, and strong shoot regeneration under defined medium compositions. Somatic embryogenesis is especially valuable because it can generate about 63 embryos per gram of callus within six weeks, shorten plantlet production by 12~15 months, and maintain high transplant establishment, thereby enabling rapid multiplication of elite lines (Figure 2) (Wang et al., 2023). However, the evidence also shows that propagation success depends strongly on explant position, developmental stage, photoperiod, temperature, sucrose concentration, and plant growth regulator regime, so the next step is not merely inventing more methods but integrating them into standardized, stage-specific propagation systems for different germplasm types (Kumar et al., 2025).
 Figure 2 Somatic embryo innovation platform for Paris polyphylla (Adopted from Wang et al., 2023) Image caption: Somatic embryos grown on medium (A, C) compared with stronger growth on filter paper+medium (B, D) (Adopted from Wang et al., 2023) |
4.3 Quality control and standardized production of artificial germplasm
Artificial germplasm restoration cannot be judged by survival and multiplication alone; it must also ensure stable medicinal quality, especially for steroidal saponins, which are the main active constituents of Paris spp. (Thapa et al., 2022; Kumar et al., 2025). A central quality-control challenge is that interspecific hybridization and morphological similarity can reduce uniformity of medicinal raw materials and complicate seed-based breeding, making genotype authentication essential (Wang et al., 2023). Molecular-marker systems linked to diversity structure and polyphyllin biosynthesis therefore provide an important foundation for quality-oriented breeding, accession identification, and traceable production (Oliya et al., 2023). At the same time, clonal systems help preserve the natural morphology and active-ingredient profiles of elite wild founders, offering a practical route to homogeneous medicinal germplasm. Standardized production should therefore integrate authenticated founder selection, clonal multiplication, and batch-level chemical evaluation rather than relying on unverified mixed-origin planting stocks (Gao et al., 2022).
Chemical evidence shows that quality in cultivated Paris is strongly shaped by plant age, culture conditions, and soil management, so standardized production must define these variables explicitly (Wang and Li, 2018; Zhang et al., 2025). Multiple studies found that major steroidal saponins vary with cultivation year and generally peak around the seventh or eighth year, with one UHPLC-MS/MS study reporting a maximum of (22.65±1.65) mg/g in the eighth year and recommending harvest at year 7 or 8. In vitro systems also affect chemical quality: mini-rhizome cultures showed 1.41-fold higher total steroidal saponins than field rhizomes under one BAP treatment, and salicylic-acid elicitation increased total saponins to 3.6 times the in vivo level, although growth slowed under elicitation. Field management also matters, because biochar and organic fertilizer significantly increased total saponin, polyphyllin I, II, VI, and VII contents through linked changes in soil nutrients, enzyme activity, and microbial communities (Liu et al., 2024). Taken together, standardized artificial germplasm production in Paris spp. should be built around authenticated elite lines, stage-specific propagation protocols, defined cultivation years, and chemical quality benchmarks supported by chromatographic and metabolomic evaluation.
5 Ecological Adaptation-Based Models for Paris spp. Germplasm Restoration
5.1 Integrated model of wild resource conservation and artificial propagation
An ecological adaptation-based restoration model for Paris spp. should begin by coupling in situ protection of wild populations with targeted artificial propagation, because wild populations remain genetically valuable but are increasingly threatened by overcollection, habitat fragmentation, and slow natural renewal (Su et al., 2022; Thakur et al., 2023). This integrated approach is supported by studies showing that cultivation is already a major route for conserving and sustainably using wild P. polyphylla var. yunnanensis, while in situ and ex situ measures are both necessary for long-term persistence. Population genetic work further indicates that wild germplasm should not be collected indiscriminately, because wild populations retain clear geographic structure and some regions, especially Guizhou and parts of Sichuan and western Yunnan, contain higher-diversity lineages that are better treated as priority conservation and provenance-selection zones (Huang et al., 2019; Yan et al., 2024). SSR analyses in Nepal likewise show that most variation occurs within populations, but germplasm from similar geographic origins clusters together, supporting region-specific conservation sampling and core germplasm construction rather than mixed, undocumented transfer (Oliya et al., 2023).
Within that framework, artificial propagation should serve as a buffer against harvest pressure and as a renewal tool for selected wild founders rather than a replacement for wild conservation. Reviews and field studies agree that in vitro propagation, ex situ cultivation, and ecologically informed niche-based planning can reduce unorganized collection from natural habitats and help design more effective conservation programs (Kunwar et al., 2020; Rawat et al., 2023). Somatic embryogenesis and related clonal systems are especially suited to this model because they can rapidly multiply elite wild accessions, preserve morphology and active-ingredient profiles, and produce plantlets with about 94% survival after transplanting to soil (Wang et al., 2023). Other regeneration platforms, including mini-rhizome production, also provide conservation-ready planting stock, with more than 95% acclimatization success and increased steroidal saponin content relative to field-grown rhizomes. The most defensible integrated model is therefore a closed loop: identify and protect high-value wild populations, select elite accessions from them, propagate those accessions under controlled conditions, and use the propagated material to supply cultivation systems and, where appropriate, reinforce depleted populations.
5.2 Combined model of understory ecological cultivation and germplasm expansion
A second restoration pathway is a combined model of understory ecological cultivation plus germplasm expansion, which fits the basic ecology of Paris spp. better than open-field domestication. Multiple ecological studies show that P. polyphylla grows and reproduces best in moist, humus-rich, well-drained forest soils under more than 80% canopy cover, with disturbed habitats supporting thinner populations and poorer regeneration. Light conditions are especially important, because less than 50% shade markedly reduces seed productivity, and the species shows poor adaptability to altered environments and climatic stress during reproduction. This explains why Nepal-based distribution and conservation work recommends conserving the species in forests and cultivating it in forest fringe areas across its potential range, rather than separating production completely from its ecological niche (Kunwar et al., 2020). Distribution modeling also indicates that ecological niches differ among medicinally used taxa, with P. polyphylla var. chinensis and var. yunnanensis responding differently to precipitation, temperature range, and human disturbance, so understory expansion should be matched to taxon-specific suitable zones rather than generalized across all planting areas (Wang et al., 2026).
Understory cultivation is not only a habitat-matching strategy; it also appears to support better medicinal chemistry under appropriate conditions. Metabolomic comparison of plants maintained for eight years under natural forest and greenhouse conditions found that naturally forest-grown roots were enriched in steroidal saponins, flavonoids, flavonols, lipids, vitamins, and veratramine alkaloids, supporting a strong association between growth environment and secondary metabolite accumulation (Yan et al., 2024). Even within understory systems, forest type matters: imitation-wild cultivation under Chinese fir and mixed forests generated higher soil organic carbon, microbial biomass carbon, water-soluble organic carbon, and enzyme activity than Moso bamboo forest, creating a more favorable soil microenvironment for P. polyphylla growth (Zhang et al., 2026). Community-level work in Arunachal Pradesh further shows that the species persists within diverse associated herb layers and that identifying such supportive ecosystems can guide conservation-oriented cultivation placement (Kalita et al., 2026). The practical implication is that germplasm expansion should use forest-compatible, site-screened understory systems that mimic native shade, litter, and soil conditions, because these systems better align with both species ecology and the formation of medicinally valuable metabolites (Rawat et al., 2023).
5.3 Germplasm renewal and industrial utilization model
The third pathway is a germplasm renewal and industrial utilization model in which elite lines are continuously renewed, authenticated, and routed into standardized production systems. This is necessary because the pharmaceutical value of Paris depends mainly on rhizome-derived steroidal saponins and polyphyllins, while current market demand continues to rise faster than wild or conventionally propagated supply (Qiang et al., 2020; Su et al., 2022). Germplasm renewal cannot rely on morphology alone, because interspecific hybridization and weak differentiation between some wild and cultivated materials can compromise raw-material uniformity and obscure breeding identity (Wang et al., 2023). Molecular infrastructure is therefore part of the renewal model itself. EST-SSR markers linked to polyphyllin biosynthesis, SSR population analysis, comparative barcoding, and dedicated biomolecular databases such as PPDP all provide tools to authenticate germplasm, trace origin, and connect genotype with medicinal-quality traits (Gao et al., 2022; Oliya et al., 2023; Wang et al., 2026). This matters for industry because traceable cultivated supply chains have already been recommended as a way to distinguish cultivated from wild-harvested stocks and support ex situ conservation without masking continued wild extraction (Rawat et al., 2023).
Industrial utilization also requires that germplasm renewal be tied to production-stage quality control, not just multiplication speed. Clonal propagation of selected elite wild accessions has already shown that candidate cultivars can be reproduced at scale while preserving morphology and active-ingredient contents, and field-grown clonal lines reached their greatest biomass increase and exceeded pharmaceutical-use polyphyllin requirements by the fifth year (Wang et al., 2023). Growth environment and management further shape industrial value. Elevated CO2 responses differed between cultivars from different natural habitats, with the western Yunnan cultivar showing stronger growth and maintained total saponin content, which suggests that renewal programs should match cultivar origin to future cultivation environments (Qiang et al., 2020). Rhizosphere engineering also appears promising: Pseudomonas palleroniana P6 increased root biomass, polyphyllin I, II, and VII content, and soil available potassium, indicating that industrial germplasm systems can be strengthened by microbe-assisted cultivation (Wu et al., 2025). Taken together, the renewal-utilization model should connect elite germplasm screening, marker-based authentication, clonal renewal, ecological site matching, and traceable downstream cultivation so that Paris spp. production shifts from wild-resource mining to adaptive, quality-controlled industrial regeneration (Oliya et al., 2023; Wang et al., 2026).
6 Challenges and Future Directions in Paris spp. Germplasm Restoration
6.1 Further improvement of germplasm evaluation systems
A central challenge in Paris spp. germplasm restoration is that evaluation systems remain incomplete, especially for linking population identity, geographic origin, genetic diversity, and medicinal quality into a single usable framework. Current studies show that molecular evaluation has advanced, but remains fragmented across marker types and regions. EST-SSR work in cultivated P. polyphylla var. yunnanensis found high polymorphism, high within-population diversity, low differentiation among cultivated populations, and clear admixture from two ancestral groups, indicating that existing cultivated materials are genetically mixed rather than standardized breeding stocks (Gao et al., 2022). SSR analysis in Nepal similarly showed that 74% of variation occurred within individuals in populations and only 26% among populations, while germplasms from similar geographic origins clustered together, supporting evaluation systems that combine individual-level diversity with provenance structure rather than relying on morphology alone (Oliya et al., 2023). AFLP studies in China reached a similar conclusion, with most genetic variation occurring within populations and with wild populations showing clear geographic structure, especially in Guizhou, Yunnan, and Sichuan, which supports region-prioritized germplasm assessment and provenance selection (Huang et al., 2019). Additional AFLP analysis from Yunnan also found that inter-population differentiation was relatively small and that gene flow among groups was limited, reinforcing the need to sample broadly while still preserving local lineages in evaluation programs.
The future direction is therefore not simply to add more markers, but to build a multi-dimensional germplasm evaluation system that integrates genetics, phylogeography, traceability, and source-level quality control. Phylogeographic work based on chloroplast trnL-trnF sequences detected 15 haplotypes, including wild-unique and cultivated-unique haplotypes, and identified Guizhou and western Yunnan as likely historical refugia that should be included in protection zones and core germplasm construction (Zhao et al., 2021). SCoT and SRAP markers also produced very high polymorphism in Dabie Mountain materials and were explicitly proposed as suitable tools for diversity analysis, genetic improvement, and conservation (Zhao et al., 2020). Beyond DNA markers, source-traceability systems are becoming feasible: a multi-block MIR/NIR platform distinguished seed germplasm from six Yunnan origins with 96.03% test accuracy, offering a practical route for rapid screening of excellent germplasm and source-based quality control (Li et al., 2022). At the time of the cited marker studies, complete genome and EST resources remained limited, and the field still required expanded molecular databases (Su et al., 2022).
6.2 Potential application of molecular breeding technologies
The second major future direction is the application of molecular breeding technologies to overcome the slow growth cycle, long seed dormancy, mixed genetic background, and unstable quality that limit conventional Paris improvement. Current evidence suggests that the species is well positioned for marker-assisted and genomics-assisted breeding, but the enabling resources are still emerging. The most direct Paris-specific evidence comes from EST-SSR markers related to polyphyllin backbone biosynthesis, which were developed specifically to characterize cultivated populations and were proposed as tools to facilitate marker-assisted breeding (Gao et al., 2022). That need is strengthened by the fact that cultivated populations show admixture, cross-pollination among cultivars, and little deep domestication differentiation from wild sources, which complicates parent selection and makes phenotype-only breeding inefficient (Huang et al., 2019). Recent assessment work also shows that accurate distinction between P. polyphylla var. chinensis and var. yunnanensis remains a practical issue for cultivation and quality control, but comparative genomic mini-barcodes can now separate them, providing a needed basis for taxon-specific breeding and deployment (Wang et al., 2026).
The broader breeding literature indicates that marker-assisted selection, genomic resources, and genome editing can sharply improve breeding precision, especially when traits are difficult to assess phenotypically or are strongly affected by environment. DNA markers improve the productivity and accuracy of classical breeding and can shorten the time required to release improved varieties (Hasan et al., 2021). Genomics-assisted breeding further expands this framework by integrating genotyping, phenotyping, and envirotyping, while genomic markers, reference genomes, transcriptomes, and expression profiles support genotype-phenotype analysis, trait mapping, and faster selection (Tyagi et al., 2024). However, the breeding literature also cautions that marker-assisted selection is most straightforward for simpler traits, whereas polygenic traits require new strategies, stronger genomic infrastructure, and more innovative selection schemes. For Paris spp., this means that future breeding should first prioritize development of reference genomes, denser diagnostic markers, and phenotype-linked quality traits such as polyphyllin content, stress adaptation, and dormancy behavior before genome editing or genomic selection can be applied effectively (Su et al., 2022).
6.3 Establishment of long-term resource restoration mechanisms
The third challenge is that germplasm restoration will not be durable unless it is embedded in long-term ecological and management mechanisms rather than isolated propagation projects. Across the Himalayan and Chinese literature, the same pressures recur: wild populations are vulnerable, slow-growing, destructively harvested, and affected by habitat degradation, illegal trade, and weak management guidelines (Kunwar et al., 2020). Reviews therefore converge on the need for combined in situ and ex situ conservation, while field studies add that local participation, awareness, and large-scale cultivation can reduce pressure on wild populations and support rural livelihoods (Thakur et al., 2023). Long-term mechanisms should also be spatially explicit. Nepal modeling predicted 51 suitable mid-hill and mountainous districts for future growth, and recent ensemble modeling in China showed that the suitable zones of var. chinensis and var. yunnanensis differ, are shaped by climate and human disturbance, and will change under future emissions scenarios. These results support restoration mechanisms that combine protected wild refugia, taxon-specific ecological cultivation zones, and long-horizon climate adaptation planning (Zhao et al., 2021; Wang et al., 2026).
A durable restoration model should therefore link policy, community, propagation, and monitoring into a continuous renewal system. Socio-ecological work in Nepal explicitly argues that sustainable production depends on understanding distribution, use, trade, and conservation together, while trade control requires stronger harvesting guidelines and more active community involvement (Kunwar et al., 2020). Studies from India likewise recommend placing P. polyphylla on priority cultivation lists, promoting rhizome and seed propagation, ecological niche modeling, and awareness programs, and maintaining long-term conservation through both field protection and cultivation support (Singh et al., 2026). Practical restoration infrastructure can include field gene banks, clonal trials, and seed production systems, as exploratory resource work in Northeast India reported conservation of distinct forms, vegetative clonal trials, and establishment of seed production systems for medicinal plant restoration programs. At the information level, PPDP already provides the first dedicated biomolecular database for Paris, integrating transcriptome, chloroplast, SSR, and functional analysis resources, and it is intended to expand further, making it a useful base for long-term germplasm documentation, trait mining, and restoration monitoring (Su et al., 2022).
7 Conclusions and Perspectives
Wild resource conservation remains the foundation of Paris spp. restoration because wild populations still contain the primary reservoirs of geographic, ecological, and genetic diversity needed for future breeding and provenance selection. This importance is reinforced by population studies showing clear geographic structuring in wild germplasm, with Guizhou, western Yunnan, and related regional groups retaining especially valuable diversity for protection and source selection. Wild Paris populations also form part of understory forest biodiversity, because it is an understory species associated with forest biodiversity and ecosystem stability. Yet these populations are under sustained pressure from overexploitation, habitat degradation, illegal trade, and anthropogenic disturbance, and multiple studies describe continuing decline or vulnerability across the Himalayan region and Southwest China.
Artificial restoration is equally important because dependence on wild rhizomes is not compatible with current medicinal demand or with the species’ biology. Demand for Paris rhizomes has risen sharply, annual trade volume is large, and cultivation remains the only realistic way to reduce extraction pressure while maintaining pharmaceutical supply. Artificial propagation is especially necessary because Paris has a long growth cycle, long seed dormancy, low seed germination, and frequent reliance on vegetative regeneration, all of which slow natural recovery. Recent propagation research shows that somatic embryogenesis, clonal regeneration, mini-rhizome systems, and improved vegetative techniques can produce restoration-ready material at higher speed and survival than conventional methods. The strongest conclusion from the current literature is therefore that in situ conservation and artificial restoration are complementary rather than alternative strategies, and sustainable utilization depends on linking the two.
Future germplasm innovation in Paris spp. will depend first on better evaluation and identification systems that connect provenance, genetic background, and medicinal quality. Existing evidence shows that cultivated populations often derive from mixed provenances and contain substantial admixture and gene flow, which complicates variety identification and quality consistency. This problem is intensified by interspecific hybridization and morphological similarity among taxa, which can reduce the uniformity of medicinal raw materials and weaken seed-based breeding. Future work should therefore integrate AFLP, SSR, EST-SSR, SCoT, SRAP, chloroplast haplotypes, and species-specific barcodes into a more complete germplasm evaluation framework. Molecular infrastructure is beginning to support that transition, as PPDP already provides the first dedicated biomolecular database for Paris and is designed to expand with additional genomic resources.
Sustainable utilization will also require breeding and cultivation systems that are ecologically adaptive and quality-oriented rather than focused on multiplication alone. Environmental conditions strongly shape both performance and metabolite accumulation in Paris, with naturally forest-grown plants showing enrichment of steroidal saponins and related metabolites relative to greenhouse-grown plants. Suitable cultivation zones also differ between var. chinensis and var. yunnanensis, and future climate and human disturbance are expected to shift those zones, making taxon-specific ecological planning increasingly important. At the production level, microbial inoculants, in vitro mini-rhizome culture, and elite clonal propagation all show potential to increase biomass and polyphyllin accumulation while supplying standardized planting stocks. Long-term restoration mechanisms should therefore combine protected wild source populations, traceable cultivated supply chains, community participation, stricter harvest governance, and continued innovation in propagation and molecular breeding.
Conflict of Interest Disclosure
The author affirms that this research was conducted without any commercial or financial relationships that could be construed as a potential conflict of interest.
Cunningham A.B., Brinckmann J.A., Bi Y.F., Pei S.J., Schippmann U., and Luo P., 2018, Paris in the spring: A review of the trade, conservation and opportunities in the shift from wild harvest to cultivation of Paris polyphylla (Trilliaceae), Journal of Ethnopharmacology, 222: 208-216.
https://doi.org/10.1016/j.jep.2018.04.048
Ding Y.G., Zhao Y.L., Zhang J., Zuo Z.T., Zhang Q.Z., and Wang Y.Z., 2021, The traditional uses, phytochemistry, and pharmacological properties of Paris L. (Liliaceae): A review, Journal of Ethnopharmacology, 278: 114293.
https://doi.org/10.1016/j.jep.2021.114293
Gao X., Su Q., Yao B., Yang W., Ma W., Yang B., and Liu C., 2022, Development of EST-SSR markers related to polyphyllin biosynthesis reveals genetic diversity and population structure in Paris polyphylla, Diversity, 14(8): 589.
https://doi.org/10.3390/d14080589
Hasan N., Choudhary S., Naaz N., Sharma N., and Laskar R.A., 2021, Recent advancements in molecular marker-assisted selection and applications in plant breeding programmes, Journal of Genetic Engineering and Biotechnology, 19(1): 128.
https://doi.org/10.1186/s43141-021-00231-1
Huang Y., Zhou N., Yang M., Shen Y., and Zhang D., 2019, A comparative study of the population genetics of wild and cultivated populations of Paris polyphylla var. yunnanensis based on amplified fragment length polymorphism markers, Ecology and Evolution, 9(18): 10707-10722.
https://doi.org/10.1002/ece3.5589
Jiang Y., Miao Y.J., Qian J., Zheng Y., Xia C.L., Yang Q., Liu C., Huang L., and Duan B., 2022, Comparative analysis of complete chloroplast genome sequences of five endangered species and new insights into phylogenetic relationships of Paris, Gene, 833: 146572.
https://doi.org/10.1016/j.gene.2022.146572
Kalita B., Sarma K., Bawri A., and Tanti B., 2026, Assessing population density and regeneration potential of Paris polyphylla Sm. in the Arunachal Himalaya, India: implications for conservation, Vegetos, 39(1): 181-192.
https://doi.org/10.1007/s42535-024-01087-9
Kumar R., Das S.P., Choudhury B.U., Kumar A., Prakash N.R., Verma R., Chakraborti M., Devi A.G., Bhattacharjee B., Das R., Das B., Devi H.L., Das B., Rawat S., and Mishra V.K., 2024, Advances in genomic tools for plant breeding: harnessing DNA molecular markers, genomic selection, and genome editing, Biological Research, 57: 80
https://doi.org/10.1186/s40659-024-00562-6
Kumar V., Sharma R., Sharma P., Sharma Y.P., Thakur K., and Sharma R., 2025, Developmental stage significantly affects in vitro propagation practices: a case study in Paris polyphylla Smith, an important endangered medicinal plant of Himalayas, Journal of Plant Growth Regulation, 44(7): 3635-3659.
https://doi.org/10.1007/s00344-025-11636-4
Kunwar R.M., Adhikari Y.P., Sharma H.P., Rimal B., Devkota H.P., Charmakar S., Acharya R.P., Baral K., Ansari A.S., Bhattarai R., Thapa-Magar S., Paudel H.R., Baral S., Sapkota P., Uprety Y., LeBoa C., and Jentsch A., 2020, Distribution, use, trade and conservation of Paris polyphylla Sm. in Nepal, Global Ecology and Conservation, 23: e01081.
https://doi.org/10.1016/j.gecco.2020.e01081
Lepcha D.L., Pradhan A., and Chhetri D.R., 2019, Population assessment and species distribution modeling of Paris polyphylla in Sikkim Himalaya, India, Biodiversitas, 20(5): 1299-1305.
https://doi.org/10.13057/biodiv/d200508
Li S., Liu C., Cai C., Wang Y., and Xu F., 2022, Geographical traceability of germplasm resources of Paris polyphylla var. yunnanensis based on multi-block information integration platform, Journal of Applied Research on Medicinal and Aromatic Plants, 31: 100440.
https://doi.org/10.1016/j.jarmap.2022.100440
Liu S., Chen Y., Li X., Lv J., Yang X., Li J., Bai Y., and Zhang S., 2024, Linking soil nutrients, microbial community composition, and enzyme activities to saponin content of Paris polyphylla after addition of biochar and organic fertiliser, Chemosphere, 363: 142856.
https://doi.org/10.1016/j.chemosphere.2024.142856
Lyngdoh M.K., Chettri A., Adhikari D., and Barik S.K., 2018, Metapopulation modelling of threatened plants to assess conservation status and determine minimum viable population size, Current Science, 114(3): 532-538.
https://doi.org/10.18520/cs/v114/i03/532-538
Oliya B.K., Maharjan L., and Pant B., 2023, Genetic diversity and population structure analysis of Paris polyphylla Sm. revealed by SSR marker, Heliyon, 9(7): e18230.
https://doi.org/10.1016/j.heliyon.2023.e18230
Puwein A., and Thomas S.C., 2019, A suitable vegetative propagation technique for effective fruiting and conservation of a vulnerable medicinal plant, Paris polyphylla Sm., Medicinal Plants-International Journal of Phytomedicines and Related Industries, 11(4): 475-480.
https://doi.org/10.5958/0975-6892.2019.00062.5
Puwein A., and Thomas S.C., 2022, Effect of plant growth regulators on in vitro propagation of Paris polyphylla, Journal of Herbs, Spices and Medicinal Plants, 28(2): 206-216.
https://doi.org/10.1080/10496475.2022.2045416
Qiang Q., Gao Y., Yu B., Wang M., Ni W., Li S., Zhang T., Li W., and Lin L., 2020, Elevated CO2 enhances growth and differentially affects saponin content in Paris polyphylla var. yunnanensis, Industrial Crops and Products, 147: 112124.
https://doi.org/10.1016/j.indcrop.2020.112124
Rawat J.M., Pandey S., Rawat B., Rai N., Preeti P., Thakur A., Butola J.S., and Bachheti R.K., 2023, Traditional uses, active ingredients, and biological activities of Paris polyphylla Smith: A comprehensive review of an important Himalayan medicinal plant, Journal of Chemistry, 2023(1): 7947224.
https://doi.org/10.1155/2023/7947224
Singh N.B., Devi L.G., Konthoujam N., Keithellakpam O.S., Thounaojam R.S., and Singh T.B., 2026, Population assessment and conservation of Paris polyphylla, a threatened medicinal plant in North East India, International Journal of Environment and Climate Change, 16(6): 316-326.
https://doi.org/10.9734/ijecc/2026/v16i65495
Su Q., Zhang X., Li J., Yang W., Ren Q., Gao X., and Liu C., 2022, PPDP: A data portal of Paris polyphylla for polyphyllin biosynthesis and germplasm resource exploration, Diversity, 14(12): 1057.
https://doi.org/10.3390/d14121057
Tang Z., Zhao J., Yang B., Sun S., Xu F., and Wang Z., 2022, Dynamic RNA-Seq study reveals the potential regulators of seed germination in Paris polyphylla var. yunnanensis, Plants, 11(18): 2400.
https://doi.org/10.3390/plants11182400
Tariq M., Nandi S.K., Bhatt I.D., Bhavsar D., Roy A., and Pande V., 2021, Phytosociological and niche distribution study of Paris polyphylla Smith, an important medicinal herb of Indian Himalayan region, Tropical Ecology, 62(2): 163-173.
https://doi.org/10.1007/s42965-020-00125-2
Thakur U., Shashni S., Thakur N., Rana S.K., and Singh A., 2023, A review on Paris polyphylla Smith: a vulnerable medicinal plant species of a global significance, Journal of Applied Research on Medicinal and Aromatic Plants, 33: 100447.
https://doi.org/10.1016/j.jarmap.2022.100447
Thapa C.B., Paudel M.R., Bhattarai H.D., Pant K.K., Devkota H.P., Adhikari Y.P., and Pant B., 2022, Bioactive secondary metabolites in Paris polyphylla Sm. and their biological activities: A review, Heliyon, 8(2): e08982.
https://doi.org/10.1016/j.heliyon.2022.e08982
Tyagi A., Mir Z.A., Almalki M.A., Deshmukh R., and Ali S., 2024, Genomics-assisted breeding: A powerful breeding approach for improving plant growth and stress resilience, Agronomy, 14(6): 1128.
https://doi.org/10.3390/agronomy14061128
Wang M., Chen J., Zhang X., Li S., Zhang T., Li W., and Lin L., 2021, Gibberellin A3 induces polyaerial shoot formation and increases the propagation rate in Paris polyphylla rhizomes, Industrial Crops and Products, 167: 113511.
https://doi.org/10.1016/j.indcrop.2021.113511
Wang M., Li W., Qiang Q., Ma J., Chen J., Zhang X., Jia Y., Zhang T., and Lin L., 2023, Clonal propagation and assessment of biomass production and saponin content of elite accessions of wild Paris polyphylla var. yunnanensis, Plants, 12(16): 2983
https://doi.org/10.3390/plants12162983
Wang Y., Liu H., Zhao D., Wang S., Wang J., Chi X., Zhang C., Wang T., Lyu C., Kang C., Sun J., Guo L., and Huang L., 2026, Assessment of suitable cultivation area for Paris polyphylla var. chinensis and var. yunnanensis under anthropogenic disturbance based on ensemble modeling and germplasm identification, BMC Plant Biology, 26(1): 241.
https://doi.org/10.1186/s12870-025-08010-7
Wang Y.Z., and Li P., 2018, Effect of cultivation years on saponins in Paris polyphylla var. yunnanensis using ultra-high liquid chromatography-tandem mass spectrometry and Fourier transform infrared spectroscopy, Plant Growth Regulation, 84(2): 373-381.
https://doi.org/10.1007/s10725-017-0348-2
Wu X., Li S., Deng Y., Duan Z., Li Y., Jiang L., Liu X., Fu S., and Liang Y., 2025, Multi-omics and field experiments reveal the mechanism of Pseudomonas palleroniana P6 promoting the growth and polyphyllins accumulation in Paris polyphylla, BMC Plant Biology, 25(1): 1214.
https://doi.org/10.1186/s12870-025-07168-4
Yan X., Wang D., Zhang A., Xia J., Jiao J., Ghanim M., Ou X., He X., and Shi R., 2024, Understory growth of Paris polyphylla accumulates a reservoir of secondary metabolites of plants, Frontiers in Microbiology, 15: 1400616.
https://doi.org/10.3389/fmicb.2024.1400616
Ye X., Tao Y., Pu X.L., Hu H., Chen J., Tan C.L., Tan X., Li S.H., and Liu Y., 2025, The genus Paris: a fascinating resource for medicinal and botanical studies, Horticulture Research, 12(3): uhae327.
https://doi.org/10.1093/hr/uhae327
Zhang H., Liu S., Zhang S., and Bai Y., 2026, Positive microbial-enzyme feedbacks on soil organic carbon enhance understory cultivation of Paris polyphylla across forest types, Land Degradation and Development, 37(9): 4189-4204.
https://doi.org/10.1002/ldr.70367
Zhang X., Chen J., Xu P., Zhang X., Yang S., Zhang J., Wan X., Gao Y., and Zheng G., 2025, Transcriptomics and metabolomics profiling of Paris polyphylla var. yunnanensis with different growth years, Scientific Data, 12(1): 866.
https://doi.org/10.1038/s41597-025-05242-y
Zhao J.J., Huang Y., Zhang D.Q., and Zhou N., 2021, Phylogeography of Paris poliphylla var. yunnanensis based on chloroplast gene trnL-trnF sequences, Zhongguo Zhong Yao Za Zhi (China Journal of Chinese Materia Medica), 46(5): 1094-1101.
https://doi.org/10.19540/j.cnki.cjcmm.20201011.102
Zhao X., Zou G., Zhao J., Hu L., Lan Y., and He J., 2020, Genetic relationships and diversity among populations of Paris polyphylla assessed using SCoT and SRAP markers, Physiology and Molecular Biology of Plants, 26(6): 1281-1293.
https://doi.org/10.1007/s12298-020-00808-z


. FPDF(win)
. FPDF(mac)
. HTML
. Online fPDF
Associated material
. Readers' comments
Other articles by authors
. Chuchu Liu

Related articles
. Paris spp.
. Wild resource decline
. Artificial germplasm
. Germplasm conservation
. Propagation
Tools
. Post a comment