Research Insight
Construction of a Standardized Cutting Propagation and Seedling Production System for Tetrastigma hemsleyanum 

 Author Correspondence author
Medicinal Plant Research, 2026, Vol. 16, No. 4
Received: 08 Jun., 2026 Accepted: 21 Jul., 2026 Published: 08 Aug., 2026
Tetrastigma hemsleyanum Diels et Gilg is an important medicinal plant resource in China with considerable medicinal value and development potential. However, the decline of wild resources, its relatively long growth cycle, and the insufficient supply of high-quality seedlings have constrained large-scale cultivation and industrial development. Cutting propagation offers several advantages, including the preservation of elite germplasm traits, a relatively short propagation cycle, simple operation, and suitability for large-scale seedling production, making it an important approach for producing high-quality T. hemsleyanum planting material. This article focuses on the construction of a standardized cutting propagation and seedling production system for T. hemsleyanum. It analyzes shoot regenerative characteristics, adventitious root formation, and the major factors affecting rooting, and systematically summarizes key techniques involving elite mother-plant selection, cutting type and specification, collection and rooting pretreatment, rooting substrate optimization, plant growth regulator application, cutting season, and planting density regulation. Seedling management measures involving temperature, humidity, water supply, light, shading, ventilation, nutrient supply, and pest and disease control are further discussed. On this basis, a standardized seedling production framework is proposed covering hardening and transplanting of rooted cuttings, seedling quality evaluation and grading, nursery release standards, and whole-process quality traceability. In view of current limitations, including insufficient screening of elite mother plants and high-rooting materials, inconsistent technical parameters and seedling quality standards, and relatively low levels of facility-based and digitalized production, future priorities should include strengthening elite germplasm selection, improving standardized operating procedures, and promoting facility-based, large-scale, and intelligent seedling production. This article provides a reference for improving cutting propagation efficiency, ensuring a stable supply of high-quality seedlings, and promoting the sustainable utilization of T. hemsleyanum medicinal resources.
1 Introduction
Tetrastigma hemsleyanum Diels et Gilg, commonly known as Sanyeqing, is a perennial climbing vine in the Vitaceae that has long been used in Chinese folk medicine and is widely recognized as a valuable traditional medicinal plant (Ji et al., 2021). Traditional and contemporary uses center on the tuberous roots and, in some contexts, the whole herb or aerial parts, which are used to clear heat, detoxify, reduce swelling and pain, promote blood circulation, and treat conditions such as high fever, pneumonia, hepatitis, pharyngeal disorders, convulsions, and inflammatory diseases (Zhu et al., 2020; Xia et al., 2023). Modern phytochemical studies show that the species contains a wide range of bioactive constituents, including flavonoids, phenolic acids, polysaccharides, triterpenoids, steroids, and organic acids, with flavonoids and polysaccharides regarded as the representative active components. These compounds underpin broad pharmacological activities, including anti-tumor, anti-inflammatory, antioxidant, antiviral, antibacterial, antipyretic, analgesic, hepatoprotective, and immunomodulatory effects (Wang et al., 2025). Mechanistic and spectrum-effect studies further indicate that T. hemsleyanum extracts can inhibit inflammatory signaling and tumor cell proliferation, while recent work on polysaccharides suggests additional antitumor activity through immune enhancement and gut microbiota regulation (Zhou et al., 2022). Because of this combination of long-standing medicinal use and expanding modern pharmacological evidence, T. hemsleyanum is increasingly regarded as a resource plant with high economic, social, and drug-development value (Hu et al., 2021; Pang et al., 2024).
At the same time, the industrial development of T. hemsleyanum remains constrained by resource scarcity, biological characteristics, and unstable production systems. Wild resources have been heavily overexploited and are now scarce or close to extinction in some regions, and the species has been described as endangered, rare, and precious because of its medicinal value and strict ecological requirements (Pang et al., 2024). The plant usually needs 3~5 years to form medicinally usable true roots, grows slowly, and is sensitive to habitat conditions such as shade and temperature, all of which limit rapid supply expansion (Zhu et al., 2020; Wang et al., 2023). Demand, however, continues to increase because the tuberous roots is the most valuable medicinal organ and the plant is already cultivated on a large scale in some areas, although its current planting modes are described as chaotic or inconsistent and the industry still lacks a scientific and measurable quality-control basis (Xia et al., 2023). Artificial cultivation has progressed over the past two decades, and greenhouse plus stereoscopic planting has been reported to improve biomass, flavonoid accumulation, yield, and overall herb quality relative to less optimized systems (Wang et al., 2025; Hu et al., 2023). Even so, the industry still faces the basic problem of producing enough uniform, high-quality planting material, which is a common bottleneck in medicinal crops and directly affects later yield, quality consistency, and resource conservation (Manohar et al., 2022; Muniandi et al., 2025).
The main propagation routes currently available for T. hemsleyanum include seed propagation, stem cutting, and tissue-culture-based rapid propagation, each with distinct practical advantages and limitations. Seed propagation offers a sexual route for population establishment, but in many medicinal plants it often produces heterogeneous offspring, and in T. hemsleyanum seed yield is already reported to be low, which limits its value for rapid industrial multiplication (Muniandi et al., 2025). Tissue culture and organogenesis can achieve high multiplication efficiency and disease-free material; for T. hemsleyanum, adventitious shoots have been regenerated from leaves and petioles, 100% rooting was achieved on media containing NAA or IBA, and acclimatized plantlets showed over 98% survival in peat:sand substrate (Pang et al., 2024). Axillary-bud rapid propagation and hairy-root systems also show strong biotechnological potential for mass propagation, conservation, and secondary metabolite production. However, tissue culture often requires specialized facilities, sterile operation, and higher costs, and in other medicinal plants it remains less accessible at farm level despite technical promise (Ioannidis et al., 2022). By contrast, cutting propagation preserves superior genotypes, enables relatively rapid and true-to-type multiplication, and is more compatible with nursery-scale and field-linked production systems. Species-specific evidence in T. hemsleyanum already shows that rooting reagent and cutting age significantly affect rooting, and that 2-3-year-old cuttings treated with 1000 mg/L IBA for 10 s gave the best tested response, providing a direct technical basis for protocol development. More broadly, studies in medicinal species show that cutting success depends on mother-stock quality, cutting position, leaf retention, season, substrate, hormone treatment, and environmental regulation, which means that the value of cuttings lies not only in the method itself but in the possibility of standardizing it into a reproducible production chain (Zhang et al., 2025; Dumani et al., 2026; Vuong et al., 2026).
This article examines the construction of a standardized cutting propagation and seedling production system for Tetrastigma hemsleyanum by integrating research findings on elite mother-plant selection, cutting material selection and specification, rooting induction, environmental regulation, seedling quality grading, and whole-process quality traceability. On this basis, the effects of mother-plant and cutting quality, rooting substrates, plant growth regulators, temperature, humidity, and light conditions on rooting and seedling establishment will be systematically analyzed, and a standardized technical pathway covering propagation material selection, rooting regulation, seedling-stage management, quality grading, and nursery release will be developed. Establishing a relatively complete cutting-based seedling production system is expected to improve propagation efficiency and seedling uniformity, reduce nursery losses, and provide high-quality planting material for the stable multiplication of elite medicinal germplasm and large-scale artificial cultivation. In addition, this article address current problems such as inconsistent propagation parameters and the lack of unified seedling quality standards, and will propose future directions toward facility-based, standardized, and digitalized nursery production. These efforts will strengthen whole-process quality control from mother-plant origin to commercial seedlings, promote coordination among germplasm conservation, standardized cultivation, and medicinal-material quality stability, and provide technical support for the sustainable utilization and high-quality industrial development of T. hemsleyanum resources.
2 Biological Basis of Cutting Propagation in Tetrastigma hemsleyanum
2.1 Shoot growth characteristics and regenerative capacity of cuttings
Tetrastigma hemsleyanum has clear regenerative potential, but current production still indicates that conventional cutting propagation yields are limited and require optimization for commercial multiplication (Pang et al., 2024). Evidence from in vitro regeneration shows that its vegetative organs retain strong organogenic competence, since leaves and petioles can regenerate adventitious shoots efficiently and axillary buds can be induced to proliferate rapidly under suitable culture conditions. This broad regenerative capacity supports the biological feasibility of building a cutting-based seedling system, because the species is not regeneration-deficient in principle but instead appears sensitive to the specification of propagule type and culture conditions.
The regenerative performance of cuttings depends strongly on the physiological status of the shoot segment, especially its age, maturity, reserve status, and nodal activity (Wei et al., 2019; Liu et al., 2025). In T. hemsleyanum, the strongest direct evidence is that 2-3-year-old cuttings rooted better than other ages, indicating that propagation material must balance juvenility with sufficient tissue maturity. Studies in other medicinal and woody species show similar positional and maturity effects: apical cuttings performed best in Chrysanthemum indicum (Ghimire et al., 2022), young apical shoots rooted better than old apical shoots in Andrographis paniculata (Hossain et al., 2021), whereas basal or middle segments in moringa often produced stronger shoots, thicker roots, or higher rooting percentages because of greater carbohydrate reserves and different endogenous hormone gradients (Muniandi et al., 2024).
2.2 Adventitious root initiation and formation in cuttings
Adventitious root formation is the developmental prerequisite for survival of detached cuttings and is therefore the core biological event in clonal propagation (Druege et al., 2019; Liu et al., 2025). In mechanistic terms, adventitious rooting is a strictly regulated process that generally proceeds through cell specification and reprogramming, primordium initiation through cell division, and primordium emergence and outgrowth (Wei et al., 2019). Tomato cutting studies further show that founder cells in basal pericycle-associated tissues first form disordered cell clusters, then dome-shaped primordia, and finally mature roots that emerge through the epidermis (Guan et al., 2019). This sequence explains why rooting speed and uniformity often vary among species and genotypes, since each stage depends on the successful completion of a distinct cellular program.
Within this program, auxin is the central regulator of adventitious rooting, while jasmonic acid, ethylene, cytokinins, and other signals modify the response (Wei et al., 2019; Liu et al., 2025). After excision, wound signaling rapidly alters hormone homeostasis, and tomato cuttings showed increased auxin and ethylene in the basal stem within 1 h, followed by auxin accumulation in meristematic founder regions and increased expression of auxin transporter genes during defined rooting phases (Guan et al., 2019). Tea and general rooting reviews likewise identify auxin as the leading hormone controlling root induction, while recent work in grape indicates that auxin and cytokinin are prominent in bud germination and leaf expansion, salicylic acid is associated with callus and root formation, and jasmonic acid and gibberellins are more closely linked to direct rooting (Wei et al., 2019; Zheng et al., 2025). In T. hemsleyanum, high rooting competence is also evident in tissue culture, where regenerated shoots formed roots at 100% frequency on media containing NAA or IBA, confirming that the species is highly auxin-responsive once suitable physiological conditions are established.
2.3 Major factors affecting rooting of cuttings
The main factors affecting rooting of T. hemsleyanum cuttings can be grouped into propagule traits, hormonal regulation, and environmental conditions, and this multifactorial control is consistent across diverse cutting systems (Campbell et al., 2021; Liu et al., 2025). For T. hemsleyanum specifically, rooting reagent and cutting age significantly affected rooting rate, whereas the tested cutting medium had no obvious effect in one study, and the best combination was 2-3-year-old cuttings treated with 1000 mg/L IBA for 10 s. More broadly, auxin type and concentration are repeatedly decisive: IBA is widely recognized as an effective rooting auxin, concentration often has the strongest effect among hormone variables (Sun et al., 2023), and excessively high levels can damage tissues and impair rooting. Species-level optima still differ, with 2 000 ppm IBA performing best in chrysanthemum (Ghimire et al., 2022), 50 ppm NAA for 30 min in Valeriana jatamansi (Gautam et al., 2021), and 3.0 mmol/L IBA accelerating rooting in young Andrographis cuttings (Hossain et al., 2021).
Environmental control is equally important because light, temperature, water status, substrate aeration, and mineral nutrition modify auxin activity, carbohydrate supply, and tissue competence for root initiation (De Almeida et al., 2017). Rooting improves when carbohydrate status is maintained, and higher light during early cultivation can offset carbohydrate depletion in cuttings, whereas low light and poor photosynthetic recovery restrict root formation (Druege et al., 2019). Light quality also matters: far-red promoted rooting in medicinal cannabis when supplied during the initial 7 d, while blue had no significant effect in that experiment . Temperature interacts strongly with auxin responses, with 25°C repeatedly supporting better root number and length than cooler or warmer conditions in chrysanthemum and tomato experimental systems (Ghimire et al., 2022; Guan et al., 2019). Substrate effects are species-dependent but often substantial: hemp rooting varied markedly across media, with substrate composition exerting the greatest effect in that study (Campbell et al., 2021), and grape cuttings rooted best in perlite or coarse-particle substrates that improved aeration (Zheng et al., 2025). Cutting diameter, leaf retention, stem wounding, humidity, season, and mother-plant health also modify rooting success by changing transpiration, endogenous hormone supply, and carbon availability.
3 Selection and Pretreatment of Cutting Materials
3.1 Selection of elite mother plants and cultivation of cutting materials
The first prerequisite for standardized cutting propagation is the selection of elite mother plants with stable phenotype, strong vegetative vigor, and high regenerative capacity, because poor stock-plant management directly lowers cutting quality. Vegetative propagation is valuable precisely because it preserves true-to-type traits from the stock plant, so the quality of the donor plant determines the quality uniformity of the seedling population (Quan et al., 2022). Mother-plant physiological status is a major determinant of rooting success, and reviews across fruit and woody crops identify it alongside cutting type, season, substrate, and hormones as a core source of variation (Saini et al., 2025). Age is especially important: hazelnut formed vigorous one-year shoots most intensively from 4-7-year-old mother plants, while younger bushes allocated more growth to plant establishment and older bushes produced weaker shoots (Savina et al., 2025). In Picea crassifolia, cuttings from 15-year-old healthy ortets showed better rooting performance than material from younger or older donor trees, indicating that optimal donor age is species-specific but biologically meaningful. Mother-plant origin also matters: tissue-culture-derived eucalyptus stock plants produced cuttings with higher rooting success and superior early growth than conventional mother-bed sources.
Elite mother plants should therefore be maintained under conditions that preserve juvenility, sanitation, and repeated shoot production. Greenhouse guidance emphasizes that healthy stock plants can tolerate frequent harvest, but they must be fully hydrated before cutting collection, and early-morning harvest is preferred because tissues are more turgid. Keeping stock plants in a juvenile state can increase the number of harvestable propagules across successive cutting rounds. Controlled mother-plant systems also improve phytosanitary quality and propagule homogeneity: soilless strawberry mother plants reduced soil-contact contamination risk and increased the quality and uniformity of propagules, while micropropagated mother plants showed substantially higher propagule output than in vivo stocks. For T. hemsleyanum, this supports establishing a dedicated mother-stock garden composed of disease-free, vigorous elite clones, managed with rejuvenation pruning, adequate water and nutrition, and protected cultivation to produce uniform juvenile shoots for repeated cutting collection (Morresi et al., 2025).
3.2 Selection of cutting types, positions, and specifications
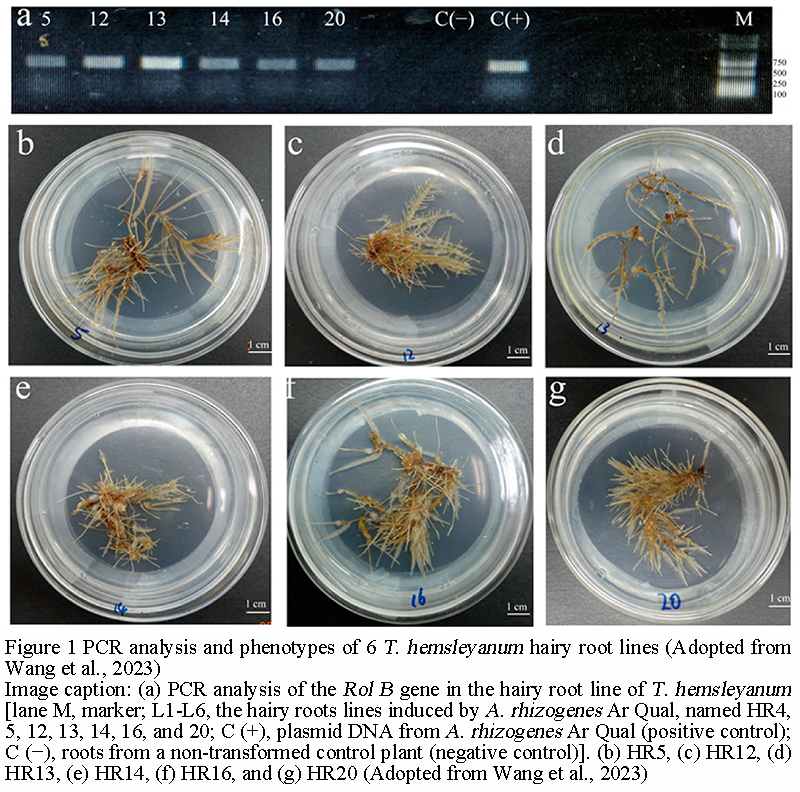
The second key step is to standardize cutting type, position, and specifications, because rooting capacity varies greatly with tissue maturity, node number, stem diameter, and topophytic origin (Figure 1) (Mohammed et al., 2020). Across many species, softwood or semi-hardwood cuttings often outperform older hardwood material. In Tecoma stans, softwood cuttings showed greater sprouting and rooting than hardwood cuttings (Singh et al., 2021). In kiwifruit, semi-hardwood cuttings produced better root traits than hardwood cuttings (Choudhary et al., 2024), and in plum rootstocks, semi-hardwood cuttings reached 100% rooting in one genotype (Seleshi et al., 2021). However, this is not universal: prairie willow rooted better from dormant hardwood than semihardwood cuttings (Schrader et al., 2026). For T. hemsleyanum, the most defensible target is physiologically juvenile but partly matured shoots, rather than highly lignified old wood or excessively succulent tissues (Saini et al., 2025). Position within the shoot also matters. Terminal stems often root faster (Singh et al., 2021), but upper-branch softwood cuttings performed best in Picea crassifolia, and basal cuttings in Prunus subhirtella produced more extensive root systems even when rooting percentage was similar to terminal cuttings. These differences reflect hormone and stress gradients after severance, so the selected cutting position should be defined empirically rather than assumed (Kunc et al., 2026).
|
Figure 1 PCR analysis and phenotypes of 6 T. hemsleyanum hairy root lines (Adopted from Wang et al., 2023) Image caption: (a) PCR analysis of the rol B gene in the hairy root line of T. hemsleyanum [lane M, marker; L1-L6, the hairy roots lines induced by A. rhizogenes Ar Qual, named HR4, 5, 12, 13, 14, 16, and 20; C (+), plasmid DNA from A. rhizogenes Ar Qual (positive control); C (−), roots from a non-transformed control plant (negative control)]. (b) HR5, (c) HR12, (d) HR13, (e) HR14, (f) HR16, and (g) HR20 (Adopted from Wang et al., 2023) |
Standardization also requires defining stem size and nodal specification. Tea softwood cuttings commonly use semi-lignified branches at least 15 cm long, while apple rootstock cuttings were standardized at 20 cm length, 5~10 mm thickness, and 4~6 buds. Tecoma cuttings were trimmed to 10 cm and 0.5~1.0 cm diameter (Singh et al., 2021), and Picea crassifolia likewise performed well with softwood cuttings 0.5~1.0 cm in diameter. Single-node cuttings can maximize propagation efficiency, but they may root slowly or fail to produce shoots in some species (Schrader et al., 2026), whereas four-node terminal semi-hardwood cuttings are used successfully in camellia. Leaf retention is also critical. Leafy cuttings rooted and sprouted better than leafless cuttings in Tecoma stans, likely because retained leaves continued photosynthesis during propagation. For T. hemsleyanum, a practical standard is to use vigorous current-season or semi-lignified shoots of moderate thickness, retain a limited functional leaf area, and specify a stable range of node number, length, and diameter to balance carbon supply with water loss (Choudhary et al., 2024).
3.3 Collection, trimming, and rooting pretreatment of cuttings
The final step is the collection, trimming, and rooting pretreatment of cuttings before insertion. Clean handling begins at harvest: stock plants should be well hydrated, cuttings should be taken in the early morning, and tools and hands should be disinfected to reduce contamination. Several studies also used fungicidal sanitation before hormone treatment, including 0.2% Bavistin for 10 min in Tecoma stans and Rizolex at 3 g/L for 5 min in fig cuttings (Singh et al., 2021). Trimming is usually standardized around the basal node, because nodes are common sites of adventitious root formation, and basal cut pattern can influence rooting depending on species (Mohammed et al., 2020). In tea, excess leaves 3~5 cm above the base were removed before sticking in perlite, while general greenhouse guidance recommends each cutting retain several leaves rather than becoming excessively leggy. Pretreatments that wound the basal region can improve rooting in some species by stimulating root initials or enhancing auxin responsiveness. Basal longitudinal or unilateral wounding was applied successfully in fig, apple rootstock, and camellia, and wounded apple cuttings showed better root and shoot parameters than unwounded ones. The effect is not universal, however, because bottle brush showed no wounding effect by itself (Hameed and Adil, 2019).
Auxin pretreatment is the most consistent rooting intervention, but concentration and application method must be standardized by species and cutting type. Quick-dip basal treatments are widely used, including 15 s in apple rootstock, short basal dips in fig, talc formulations in Tecoma stans, and 5 min immersion or 15 s basal dip in camellia. IBA repeatedly outperformed or matched other auxins, with optimal reported concentrations of 1000 mg/L in catalpa (Quan et al., 2022), 2 000 ppm in apple rootstock, and 0.4% IBA in Tecoma stans (Singh et al., 2021). Auxin combinations can further improve rooting in some species, as in magnolia with NAA:IBA (2:1) and fig with wounding plus IBA and NAA. Because T. hemsleyanum needs a reproducible nursery protocol, its cuttings should be harvested from hydrated elite mother plants, disinfected, trimmed to a fixed nodal and leaf standard, optionally wounded at the base, and subjected to a calibrated IBA-based quick-dip treatment before insertion into the rooting substrate.
4 Optimization of Key Techniques for Rooting of Cuttings
4.1 Selection and optimization of rooting substrates
The rooting substrate should first satisfy the physical requirements of water retention plus aeration, because adventitious rooting responds strongly to pore structure, oxygen availability, and moisture balance rather than to any single substrate ingredient (Hoover et al., 2025; Saini et al., 2025). Across species, mixed media often outperform single materials when they balance these properties, as peat+perlite outperformed perlite alone in Caucasian whortleberry and cocopeat+perlite (1:1) gave optimum rooting in carnation (Yazar et al., 2025). Similar advantages appear in woody and succulent systems, where perlite-cocopeat (1:1) gave the best juniper protocol and sand:perlite or sand:vermiculite supported the highest rooting percentage and root number in Pedilanthus tithymaloides (Abass et al., 2024). In chrysanthemum, vermiculite+perlite (1:1) supported the best response under the optimal auxin-temperature combination, again indicating that porous, well-aerated mixtures are broadly favorable for cutting propagation (Ghimire et al., 2022).
At the same time, the best substrate remains species-dependent, so standardization for T. hemsleyanum should define a preferred range of structure rather than assume one universal medium (Zheng et al., 2020; Mello et al., 2025). Some species root best in highly aerated coarse media, as grape cuttings rooted best in pure perlite and in other large-particle substrates such as coarse sand mixtures (Zheng et al., 2025). Others favor alternative materials, such as Kanuma soil in Apocynum lancifolium, which gave the highest survival and rooting rate among the tested substrates (Seo et al., 2023). Substrate design also has to consider later plug quality, because stratifying peat-based media with coarse amendments did not clearly improve root growth but reduced plug structural stability in herbaceous cuttings (Hoover et al., 2025). For T. hemsleyanum, the most defensible standard is therefore a clean, moderately fine but aerated substrate, with perlite-based or peat/cocopeat-perlite mixtures prioritized for rooting trials and plug integrity evaluated together with rooting percentage, root length, and root biomass (Abshahi et al., 2022).
4.2 Types, concentrations, and application methods of plant growth regulators
Among plant growth regulators, IBA is the most consistently effective rooting auxin across cutting systems, although the optimum dose varies by species, cutting type, and physiological state (Seo et al., 2023; Saini et al., 2025). IBA improved rooting percentage, root number, root length, and root quality in juniper, chrysanthemum, guava, bottle brush, dragon fruit, and Solanum procumbens, with species-specific optima ranging from 500 to 3 000 ppm (Abshahi et al., 2022; Marappan et al., 2026). In T. hemsleyanum, the direct evidence points to 1000 mg/L IBA for 10 s as the best tested treatment, which is notably consistent with the 1 000 ppm optima reported in juniper, catalpa, and bottle brush (Quan et al., 2022; Muniandi et al., 2025). Mechanistically, exogenous auxin promotes cell division, assimilate mobilization, root primordium differentiation, and favorable endogenous hormone ratios such as higher IAA/ABA and IAA/ZR, which together accelerate root initiation and improve uniformity (Abass et al., 2024).
However, more auxin is not always better, and several studies show a threshold beyond which rooting declines or root systems become short and coarse (Ghimire et al., 2022). In carnation, rooting percentage did not increase with increasing auxin concentration, and higher concentrations inhibited rooting (Zheng et al., 2020). In Apocynum lancifolium, Rootone gave the highest rooting rate, while 500~1000 mg/L IBA reduced survival relative to lower-dose or control treatments, despite 1000 mg/L producing more roots (Seo et al., 2023). By contrast, some species require higher IBA doses, including 3 000 ppm in dragon fruit and 3 000 ppm in guava single-node cuttings, while ivy gourd responded best to 1 500 ppm IBA and Solanum procumbens to 500 ppm (Jayaganesh et al., 2025; Choudhary et al., 2026). Combined auxin treatments can also be useful in some systems, since IBA+NAA improved rooting in carnation and dragon fruit, but IBA alone still outperformed NAA in catalpa and bottle brush (Marappan et al., 2026). For T. hemsleyanum, the present evidence supports adopting a short basal dip in IBA as the standard core treatment, then refining concentration by cutting age and season rather than broadly increasing dose (Saini et al., 2025).
4.3 Regulation of cutting time, planting depth, and density
The timing of cutting collection should match periods of high physiological activity but moderate stress, because season strongly affects rooting capacity, sprouting, and subsequent seedling growth (Seo et al., 2023). Across species, spring and early autumn repeatedly perform well: juniper rooted best in spring, tea cuttings performed best when collected from early September to late October, bamboo rooted best in spring-summer, and camellia showed higher survival and bud sprouting in spring and autumn than in summer or winter (Abshahi et al., 2022; Kumar et al., 2022). Caucasian whortleberry also showed its highest rooting in September with semi-hardwood cuttings, while cerrado pitaya performed better in spring and was not recommended for autumn preparation (Yazar et al., 2025; Mello et al., 2025). Reviews of fruit-cutting propagation similarly conclude that early planting, especially February-March, often enhances rooting because carbohydrate accumulation is more favorable (Saini et al., 2025). For T. hemsleyanum, this supports scheduling propagation in spring or early autumn and avoiding periods of extreme summer heat or deep winter dormancy.
Cutting specification and planting layout should also be standardized, because rooting varies with shoot position, cutting size, node number, and likely with insertion geometry and crowding (Kumar et al., 2022). Mid or basal shoot portions often perform better than top portions, as shown in tea and moringa, although apical sections can perform best in some species such as chrysanthemum, confirming that positional effects are real but genotype-specific (Ghimire et al., 2022). Cutting size also shows a consistent trade-off: medium diameters gave the best overall efficiency in camellia, thicker cuttings improved rooting in one bamboo species, and moringa showed that larger cuttings favor shoot growth whereas smaller ones favor root initiation (Muniandi et al., 2025). Single-node cuttings can maximize propagation efficiency when stock is limited, as shown in tea and guava, provided leaf area and humidity are sufficient to avoid desiccation stress. Direct evidence on planting depth and density is limited in the supplied literature, but the same studies indicate that resource competition, leaf retention, and cutting stability affect rooting outcomes, so T. hemsleyanum should use shallow-to-moderate insertion of the basal node region in a loose substrate and a spacing density that prevents leaf overlap, preserves aeration, and facilitates uniform misting and disease control (Seo et al., 2023).
5 Environmental Regulation and Seedling Management during Cutting Propagation
5.1 Regulation of temperature, humidity, and water supply
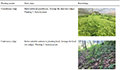
During the rooting stage of Tetrastigma hemsleyanum cuttings, temperature, humidity, and water supply should be managed as an integrated environmental unit, because high survival before root emergence depends on limiting desiccation while maintaining metabolic conditions favorable to callus formation and adventitious root initiation (Table 1) (Rock et al., 2022; Hu et al., 2023). Studies across propagation systems show that high relative humidity consistently supports rooting by reducing transpiration from unrooted shoots; in rose, 98~100% relative humidity is recommended initially and then gradually reduced, while in cannabis high humidity promoted rooting across cultivars and in forest-tree mist chambers successful rooting was maintained near 85% relative humidity (Yang et al., 2022; Kim et al., 2025; Kamara et al., 2025). Fine misting or fogging is preferred because it maintains humid air and supplies moisture without heavy wetting, whereas excessive droplet retention raises the risk of rot and mortality (Shen et al., 2025). Substrate water status also requires moderation rather than saturation: lavender cuttings showed the highest survival at about -2.5 kPa, high rooting at -1.0 to -2.5 kPa, and mortality above 50% under the driest treatment, indicating that the rooting medium should remain evenly moist but aerated until roots are established.
|
Table 1 Four planting modes of T. hemsleyanum (Adopted from Hu et al., 2023) |
Temperature control should aim at a warm and stable rooting zone while avoiding excessive heat, because both direct rooting responses and water relations deteriorate under thermal stress (De Almeida et al., 2017). In mulberry aeroponic propagation, maintaining 25~27 °C together with 90~100% humidity increased rooting by 41.40%, callusing by 58.89%, and reduced mortality by 55.85% relative to non-regulated conditions (Shen et al., 2025). Juniper cuttings rooted best when the rooting table was maintained at (25±2)°C rather than (20±2)°C (Güney et al., 2021), and microcuttings of Corymbia and Eucalyptus performed best in controlled environments where mean temperatures remained moderate, with an estimated ideal maximum of 28.4°C and minimum of 20.3°C. Temperature effects also extend to donor-plant conditioning: reduced nighttime temperature lowered rooting in Eucalyptus dunnii, decreased soluble carbohydrates at the cutting base by about 25%, and reduced foliar nutrient status, showing that stable thermal management helps preserve the physiological quality of propagation materials before and after excision (Nión et al., 2026). Therefore, T. hemsleyanum cuttings should be kept under warm, humid, and finely misted conditions, with moderate substrate moisture and careful avoidance of prolonged leaf wetness or overheating (Rock et al., 2022).
5.2 Management of light, shading, and ventilation
Light regulation during cutting propagation should balance protection from excessive radiation with maintenance of minimum photosynthetic function, because both over-shading and excessive light reduce seedling vigor through different mechanisms (Huang et al., 2025). Moderate shading often improves seedling quality in shade-sensitive or heat-stressed nursery crops. In Castanopsis hystrix, 60% shade produced the highest quality index and improved root characteristics relative to no shade, while excessive shading restricted dry matter accumulation (Xue et al., 2023). In Hopea hainanensis, 0~30% shading was most favorable overall, and a dynamic strategy of initial 30% shading followed by gradual reduction was proposed to support early establishment and later biomass partitioning. In plastic-greenhouse cultivation of Cyclocarya, shading increased survival, reduced leaf burn, and improved biomass compared with the unshaded control, which suffered inhibited growth under summer heat (Feng et al., 2023). These results indicate that T. hemsleyanum cuttings and young rooted seedlings should be protected from intense direct radiation, especially in warm seasons or enclosed facilities, but should not be maintained under chronically deep shade.
Ventilation should be coordinated with shading and humidity management rather than maximized indiscriminately, because air exchange can reduce heat accumulation and disease-favoring stagnation but may also disrupt the high-humidity microclimate required for unrooted cuttings (Ventura et al., 2019). In microcutting systems, a shade house without fogging and a greenhouse without ventilation but with fogging gave the best rooting, root growth, and survival, whereas greenhouse environments with ventilation had poorer performance and in one case higher temperatures. Heated mini-tunnels likewise improved winter rooting and physiological performance in Eucalyptus dunnii by protecting plants from low temperatures and maintaining adequate humidity, while supplemental lighting served mainly to overcome seasonal constraints rather than replace environmental conditioning (Schilisting et al., 2025). Practical regulation should therefore use shade nets or protected structures to buffer radiation and temperature, maintain gentle ventilation sufficient to renew air, and gradually increase light exposure and air movement only after rooted cuttings begin active leaf expansion (Xue et al., 2023; Shen et al., 2025).
5.3 Nutrient supply and pest and disease control during the seedling stage
After initial callus and root formation, nutrient supply becomes necessary to sustain the transition from root induction to seedling growth, but fertilization should remain balanced and stage-specific because excessive or poorly matched nutrition can impair seedlings rather than improve them (Pascual et al., 2018). In mulberry rapid propagation, only clean water was used during the first four days after insertion, after which Hoagland nutrient solution was introduced and replaced every five days in summer, illustrating the principle that nutrient supply should follow rather than precede early rooting stabilization (Shen et al., 2025). Fertilization can substantially improve cutting and seedling growth when correctly managed: NPK at 20~30 g/L increased rooting and sprouting of apical forest-tree cuttings, moderate N and P improved cocoa cutting growth, and balanced mineral nutrition is repeatedly identified as a determinant of adventitious rooting and survival (De Almeida et al., 2017). Substrate-linked nutrient strategies also matter. Cocopeat improved aeration and water-holding capacity over sterilized soil in clonal forestry cuttings, cattle-manure-containing substrates improved seedling growth and nutrient accumulation in African mahogany, and bio-inoculants such as AMF or PGPR enhanced P, K, Ca, and chlorophyll in rooted hazelnut cuttings, although nitrogen remained limiting when N supply was inadequate (Kamara et al., 2025).
Pest and disease control during the seedling stage should emphasize prevention, sanitation, and environmental regulation, because contaminated cuttings, substrates, irrigation water, and poorly ventilated wet nursery conditions allow pathogens to spread early and persist into field planting. Integrated management begins with healthy propagules and clean infrastructure: cuttings can carry surface microorganisms, so disinfection of plant material, tools, hands, containers, and substrates is essential, and contaminated media may require steam or other disinfestation measures (Shen et al., 2025). Disease suppression can also be supported biologically and culturally, since compost-based substrates may provide pathogen suppressiveness, beneficial microorganisms can improve nutrition and resistance, and irrigation, humidity, storage, and nursery hygiene all directly affect seedling health (Pascual et al., 2018). Nursery production should therefore include routine removal of diseased seedlings and residues, maintenance of irrigation-water quality, controlled access and operation records, and balanced nutrition that avoids weakening seedlings or predisposing them to infection (Ventura et al., 2019).
6 Construction of a Standardized Seedling Production System for Tetrastigma hemsleyanum
6.1 Hardening, transplanting, and establishment management of rooted cuttings
Hardening of rooted cuttings should proceed by gradual acclimatization, not abrupt transfer, because newly rooted propagules often suffer transplant shock before they become fully coupled to the field environment (Grossnickle and Macdonald, 2018). In carob, rooted cuttings were transplanted into sterilized sand:soil substrate and kept under rooting-phase conditions for four weeks before relative humidity was progressively reduced to normal greenhouse conditions, showing a practical model for staged acclimation (Essahibi et al., 2017). Comparable medicinal-plant studies also show that post-rooting hardening can determine final survival, with rooted Aphanamixis polystachya reaching 72% survival after hardening and micropropagated Alangium salviifolium achieving 60% transfer to soil after greenhouse acclimatization (Pandey et al., 2022; Gurav et al., 2025). By contrast, Ruta chalepensis plantlets survived at 95.2% after effective hardening, indicating that acclimatization quality can sharply change establishment outcomes even when rooting has already occurred (Qahtan et al., 2021).
Transplanting management should therefore prioritize root protection, gradual humidity reduction, suitable substrate transition, and early establishment vigor. Evidence across cutting systems indicates that survival after transplanting improves when rooted propagules are moved into clean, aerated substrates and maintained under moderated conditions before full field exposure (Izadi et al., 2022). Physiologically, cutting quality after rooting still depends on leaf vitality, source-sink balance, and uniform root development, and delayed or uneven rooting can impair synchronous later growth among individuals (Druege, 2020). For T. hemsleyanum, hardening should thus retain moderate shade and humidity at first, then gradually increase ventilation and reduce protection, while transplanting should use rooted cuttings with intact leaves, healthy white roots, and no basal decay so that establishment management begins from physiologically functional planting stock (Sarolia et al., 2021; Mataruga et al., 2023).
6.2 Seedling quality evaluation, grading, and nursery release standards
Seedling quality evaluation for T. hemsleyanum should combine morphological indicators with selected physiological or functional indicators, because morphology remains the operational basis of quality control, but morphology alone does not capture all differences in transplant performance. Reviews of seedling quality practice show that morphological attributes are widely used and often mandatory, while physiological attributes are used less often despite their value for monitoring crop development, nutrient status, viability, and post-planting performance (Grossnickle and Macdonald, 2018). The broader seedling-quality literature also rejects a single universal test: no “silver bullet” applies across nursery, lifting, and pre-planting stages, so quality control must use stage-appropriate indicators and explicit testing purposes. For rooted cuttings specifically, additional quality requirements apply beyond ordinary seedling stock, reinforcing the need for a dedicated standard for clonal T. hemsleyanum nursery material.
A practical grading system should be simple enough for nursery use but sufficiently predictive of later medicinal production. In Panax notoginseng, unclear seedling sources and uneven quality reduced emergence and acclimatization, and the establishment of a grading standard improved normative industry management. That study found that root length, root diameter, and bud diameter correlated positively with fresh weight, and finally simplified grading to fresh weight plus rootlet number, with higher grades showing better emergence, photosynthetic performance, and medicinal output after transplanting. Similar patterns appear in other medicinal crops: graded transplantation in Astragalus membranaceus changed both yield and active component content after transplanting, and licorice seedling grades based on plant weight produced 1.5-2-fold differences in several bioactive constituents in the harvested roots (Li et al., 2023). Accordingly, nursery release standards for T. hemsleyanum should classify rooted cuttings into at least premium, standard, and cull grades using easily measured indices such as seedling height, stem thickness, leaf number, root number, root length, root fresh weight, and root system integrity, while excluding seedlings with deformities, weak growth, pest damage, or poor plug development (Grossnickle and Macdonald, 2018; Sarolia et al., 2021).
6.3 Standardized whole-process production and quality traceability for cutting seedlings
Whole-process standardization for T. hemsleyanum should begin with the origin control of mother plants and propagules and continue through nursery management, handling, and shipping. Across European systems, control of the origin of seed and vegetative material and pest and disease status are common elements of seedling quality control (Mataruga et al., 2023). Evidence from medicinal-plant production likewise shows that mixed varieties and materials with unclear sources lead to poor field performance, unstable quality, and difficulty in supervision . Standardization also needs explicit nursery protocols for watering, shading, fertilization, growing media, root pruning, weed control, storage, transport, and handling, because these operational steps are already recognized as determinants of seedling quality (Sarolia et al., 2021). This matters especially for cuttings, since quality can decline during storage, shipping, or transition between production environments, and unsuitable transport and handling are a known cause of reduced seedling quality (Druege, 2020).
Traceability should convert that standardized process into a recorded and auditable production chain. Barcode-based in vitro seedling management systems already show that recording medium composition, culture stage, multiplication generation, and production operations can solve fragmented recordkeeping and provide a practical tool for quality control and supervision. IoT-based greenhouse traceability systems extend this principle by continuously tracking luminosity, humidity, temperature, and water consumption, while also enabling automated environmental control and internal traceability from early growth to final output. More general production frameworks likewise emphasize four linked layers: genetic integrity, field or nursery production standards, post-harvest or post-production handling and testing, and certification with traceability. Therefore, the standardized seedling production system for T. hemsleyanum should assign each cutting lot a unique identity linked to mother plant source, collection date, cutting specification, pretreatment formula, substrate batch, environmental records, rooting and hardening results, grading outcome, release destination, and any later field feedback, thereby establishing a closed-loop quality traceability system from elite mother plant to commercial seedling.
7 Current Problems and Future Directions
Insufficient selection of elite mother plants and high-rooting propagules remains a major problem, because clonal propagation only delivers stable medicinal quality when the source genotype is first screened for desirable agronomic and phytochemical traits. Studies in medicinal species show that wild collections are often heterogeneous and produce variable end products, whereas clonal lines derived from selected accessions improve uniformity of essential oil or metabolite profiles. Mother stock management is equally important, since homogeneous juvenile explants produced under controlled ex situ conditions are more suitable for protocol development than irregular materials taken directly from the wild. Evidence across medicinal and woody species also shows that rooting capacity depends on propagule type and source, including apical versus basal position, cutting girth, tissue maturity, and leaf retention, but the optimal combination is genotype-specific rather than universal. For T. hemsleyanum, this means future work should shift from general collection of mother vines toward the establishment of elite source gardens, with selection based on genotype identity, growth vigor, medicinal constituent stability, and repeatable rooting performance of defined cutting types.
The lack of unified technical parameters for cutting propagation and seedling quality evaluation, remains a recognized barrier even in other medicinal crops already under commercialization. Reviews of medicinal and aromatic plants show strong consensus that standardization of vegetative propagation is essential for cultivation, conservation, and commercial uniformity, yet rooting success still varies widely with cutting maturity, season, length, hormone concentration, substrate, and greenhouse environment. Species-specific studies illustrate how large these parameter effects can be: apical shoots outperformed basal stem cuttings in one medicinal cannabis system, apical cuttings with 2 000 ppm IBA rooted best in Chrysanthemum indicum at 25°C in vermiculite:perlite 1:1, and selected Valeriana jatamansi clones required 50 ppm NAA for 30 min with media such as sand or cocopeat for reliable large-scale multiplication. At the seedling stage, the absence of grading standards also weakens quality control, because high-quality planting material is the precondition for standardized herb production and formal grading criteria can be built around measurable vigor indices. For T. hemsleyanum, the next step is to convert current empirical experience into unified SOPs that specify mother plant age, cutting position and size, leaf retention, pretreatment formula, substrate composition, environmental set points, rooting benchmarks, and nursery release grades for qualified seedlings.
Seedling production systems remain insufficiently facility-based, large-scale, and digital, even though commercial propagation increasingly depends on controlled environments and process automation. Large-scale medicinal plant propagation has already shown that root trainers, shade structures, and multi-tier nursery layouts can sharply expand output while reducing land demand; in Valeriana jatamansi, three multiplication cycles from ten starter plants could produce about 80 000 plants, and vertical nursery arrangements could further reduce space requirements. Recent engineering studies also show that automation can improve seedling handling efficiency and reproducibility: machine-vision systems can guide robotic implantation and tray logistics, automated plug-seedling equipment can integrate sowing, covering, fertilizing, watering, and cloud-based monitoring of depth, temperature, and humidity, and smart transplanting frameworks using sensors and PLC control can reduce missed seedlings and improve operational reliability. Digital twin systems go further by linking real-time sensing, predictive modeling, simulation, and robotic execution in a closed loop, with more than 90% localization accuracy reported in greenhouse operations. For T. hemsleyanum, future development should therefore combine protected facility propagation with digital traceability, environmental monitoring, automated irrigation and mist control, and eventually intelligent transplanting and grading, so that cutting seedling production becomes not only standardized but also scalable, auditable, and less dependent on manual experience.
Conflict of Interest Disclosure
The author affirms that this research was conducted without any commercial or financial relationships that could be construed as a potential conflict of interest.
Abass M.M.M., Thabet R.S., Lasheen F.F., Abdelhamid A.N., Hassan K.M., Saudy H.S., and Boghdady M.S., 2024, Modulating the rhizosphere medium and indole-3-butyric acid supply influence rooting, nutrients and biochemical constituents and histological features of Pedilanthus tithymaloids, Journal of Soil Science and Plant Nutrition, 24(4): 6880-6892.
https://doi.org/10.1007/s42729-024-02011-5
Abshahi M., García-Morote F.A., Zarei H., Zahedi B., and Nejad A.R., 2022, Improvement of rooting performance in stem cuttings of Savin Juniper (Juniperus sabina L.) as a function of IBA pretreatment, substrate, and season, Forests, 13(10): 1705.
https://doi.org/10.3390/f13101705
Campbell S.M., Anderson S.L., Brym Z.T., and Pearson B.J., 2021, Evaluation of substrate composition and exogenous hormone application on vegetative propagule rooting success of essential oil hemp (Cannabis sativa L.), PLOS ONE, 16(7): e0249160.
https://doi.org/10.1371/journal.pone.0249160
Choudhary S., Kumar S., Yadav S., and Saini S., 2026, Effect of plant growth regulators on root development of dragon fruit cuttings (Hylocereus costaricensis Britton & Rose), Plant Archives, 26(1): 681-686.
https://doi.org/10.51470/plantarchives.2026.v26.no.1.093
Choudhary S., Rana V.S., Choudhary M., Choudhary K., Choudhary R., and Choudhary J., 2024, Evaluation of hardwood and semi-hardwood cuttings for rooting performance in exotic kiwifruit cultivars, Journal of Scientific Research and Reports, 30(10): 368-374.
https://doi.org/10.9734/jsrr/2024/v30i102464
De Almeida M.R., Aumond M. Jr., Da Costa C.T., Schwambach J., Ruedell C.M., Correa L.R., and Fett-Neto A.G., 2017, Environmental control of adventitious rooting in Eucalyptus and Populus cuttings, Trees, 31(5): 1377-1390.
https://doi.org/10.1007/s00468-017-1550-6
Druege U., 2020, Overcoming physiological bottlenecks of leaf vitality and root development in cuttings: a systemic perspective, Frontiers in Plant Science, 11: 907.
https://doi.org/10.3389/fpls.2020.00907
Druege U., Hilo A., Pérez-Pérez J.M., Klopotek Y., Acosta M., Shahinnia F., Zerche S., Franken P., and Hajirezaei M.R., 2019, Molecular and physiological control of adventitious rooting in cuttings: phytohormone action meets resource allocation, Annals of Botany, 123(6): 929-949.
https://doi.org/10.1093/aob/mcy234
Dumani A., Silwana T.T., Egbichi I., Oyedeji A.O., Mpambani B., and Seepe H.A., 2026, Effects of cutting position and leaf area retention on rooting and growth of vegetatively propagated Cannabis sativa, Journal of Applied Horticulture, 28(1): 92-97.
https://doi.org/10.37855/jah.2026.v28i01.13
Essahibi A., Benhiba L., Oussouf F.M., Ait Babram M., Ghoulam C., and Qaddoury A., 2017, Improved rooting capacity and hardening efficiency of carob (Ceratonia siliqua L.) cuttings using arbuscular mycorrhizal fungi, Archives of Biological Sciences, 69(2): 291-298.
https://doi.org/10.2298/abs160307100e
Feng Y., Zhi L., Pan H., Chen Y., and Xu J., 2023, Shade improves seedling quality of ornamental Cyclocarya species under plastic greenhouse cultivation, Ornamental Plant Research, 3: 13.
https://doi.org/10.48130/opr-2023-0013
Gautam R.D., Kumar A., Kumar R., Chauhan R., Singh S., Kumar M., Kumar D., Kumar A., and Singh S., 2021, Clonal propagation of Valeriana jatamansi retains the essential oil profile of mother plants: an approach toward generating homogenous grade of essential oil for industrial use, Frontiers in Plant Science, 12: 738247.
https://doi.org/10.3389/fpls.2021.738247
Ghimire B.K., Kim S.H., Yu C.Y., and Chung I.M., 2022, Biochemical and physiological changes during early adventitious root formation in Chrysanthemum indicum Linné cuttings, Plants, 11(11): 1440.
https://doi.org/10.3390/plants11111440
Grossnickle S.C., and MacDonald J.E., 2018, Seedling quality: history, application, and plant attributes, Forests, 9(5): 283.
https://doi.org/10.3390/f9050283
Guan L., Tayengwa R., Cheng Z., Peer W.A., Murphy A.S., and Zhao M., 2019, Auxin regulates adventitious root formation in tomato cuttings, BMC Plant Biology, 19(1): 435.
https://doi.org/10.1186/s12870-019-2002-9
Güney D., Chavoshi S.H., Bayraktar A., and Atar F., 2021, The effects of temperature and exogenous auxin on cutting propagation of some junipers, Dendrobiology, 86: 29-38.
https://doi.org/10.12657/denbio.086.004
Gurav A., Vaze G.V., Bondade P.P., Nirawane R.B., Kolhe R.H., Prasad S.B., Prasad G.P., Mathapati S.N., and Srikanth N., 2025, In vivo propagation of Aphanamixis polystachya (Wall.) R. Parker, Journal of Drug Research in Ayurvedic Sciences, 10(4): 287-294.
https://doi.org/10.4103/jdras.jdras_11_24
Hameed R.L., and Adil A.M., 2019, Effect of wounding, auxins and cinnamon extract on the rooting and vegetative growth characteristics of bottle brush plant (Melaleuca viminalis L.) cuttings, Scientific Journal of Flowers and Ornamental Plants, 6(2): 105-111.
https://doi.org/10.21608/sjfop.2020.70777
Hoover B.K., De La Cruz M.J., Whitehead E.C., and Wu A., 2025, Stratified cutting propagation substrates reduce herbaceous plug structural stability but facilitate similar root growth to a control, HortTechnology, 35(6): 910-916.
https://doi.org/10.21273/HORTTECH05739-25
Hossain M.S., Urbi Z., and Phang I.C., 2021, Auxin increased adventitious root development in the medicinal plant Andrographis paniculata (Burm. f.) Wall. ex Nees, Agronomy Journal, 113(4): 3222-3231.
https://doi.org/10.1002/agj2.20745
Hu W., Jiang M., Liang Z., and Xia P., 2023, The stereoscopic planting mode improved the quality and yield of Tetrastigma hemsleyanum, South African Journal of Botany, 157: 44-52.
https://doi.org/10.1016/j.sajb.2023.03.048
Hu W., Zheng Y., Xia P., and Liang Z., 2021, The research progresses and future prospects of Tetrastigma hemsleyanum Diels et Gilg: a valuable Chinese herbal medicine, Journal of Ethnopharmacology, 271: 113836.
https://doi.org/10.1016/j.jep.2021.113836
Huang C., Lin L., Chen F., Wang X., Shi M., Chen L., Yang X., Dong X., and Zhang M., 2025, Shading effects on the growth and physiology of endangered Hopea hainanensis Merr. and Chun seedlings, Forests, 16(7): 1193.
https://doi.org/10.3390/f16071193
Ioannidis K., Tomprou I., and Mitsis V., 2022, An alternative in vitro propagation protocol of Cannabis sativa L. (Cannabaceae) presenting efficient rooting, for commercial production, Plants, 11(10): 1333.
https://doi.org/10.3390/plants11101333
Izadi Z., Nejad R.A., and Abadía J., 2022, Iron chelate improves rooting in indole-3-butyric acid-treated rosemary (Rosmarinus officinalis) stem cuttings, Agriculture, 12(2): 210.
https://doi.org/10.3390/agriculture12020210
Jayaganesh A., Reddy P.S.S., Sadarunnisa S., Padmaja V.V., and Reddy B.H.M., 2025, Influence of type of cuttings and plant growth regulators on adventitious root formation and growth of ivy gourd (Coccinia grandis L.) cuttings, Plant Archives, 25(2): 2362-2368.
https://doi.org/10.51470/plantarchives.2025.v25.no.2.336
Ji T., Ji W.W., Wang J., Chen H.J., Peng X., Cheng K.J., Qiu D., and Yang W.J., 2021, A comprehensive review on traditional uses, chemical compositions, pharmacology properties and toxicology of Tetrastigma hemsleyanum, Journal of Ethnopharmacology, 264: 113247.
https://doi.org/10.1016/j.jep.2020.113247
Kamara E.G., Kamara P., Mattia S.B., Kassoh F.A., and Kanu S.A., 2025, Growth performance of apical and nodal cuttings of selected forest tree species under different fertilizers and substrate regimes in the nursery, European Journal of Applied Sciences, 13(5): 546-557.
https://doi.org/10.14738/aivp.1305.19530
Kim B., Hahm S., Lee Y., Bok G., and Park J., 2025, Light, temperature, and relative humidity influence the adventitious rooting of Cannabis stem cuttings, Horticultural Science and Technology, 43(4): 480-493.
https://doi.org/10.7235/hort.20250043
Kumar P., Mishra J.P., Sonkar M.K., Mishra Y., and Shirin F., 2022, Relationship of season and cuttings’ diameter with rooting ability of culm-branch cuttings in Bambusa tulda and Bambusa nutans, Journal of Plant Growth Regulation, 41: 2491-2498.
https://doi.org/10.1007/s00344-021-10461-9
Kunc P., Medic A., Grohar M.C., Mrak T., and Osterc G., 2026, Physiological maturation and hormonal profiles associated with rooting performance and root system architecture of leafy cuttings in Prunus subhirtella ‘Autumnalis’, BMC Plant Biology, 26(1): 804.
https://doi.org/10.1186/s12870-026-08644-1
Li X., Mu Y., Zhang X., and Wang J., 2023, Effects of graded seedling transplanting on growth, yield and medicinal materials quality of Astragalus membranaceus var. mongholicus, Legume Research, 46(6): 728-734.
https://doi.org/10.18805/LRF-720
Liu P., Zhang S., Wang X., Du Y., He Q., Zhang Y., Shen L., Hu H., Zhang G., and Li X., 2025, Adventitious root formation in cuttings: insights from Arabidopsis and prospects for woody plants, Biomolecules, 15(8): 1089.
https://doi.org/10.3390/biom15081089
Manohar K.A., Shukla G., Roy B., and Chakravarty S., 2022, Effects of plant growth regulators and growing media on propagation and field establishment of Stevia rebaudiana: a medicinal plant of commerce, CABI Agriculture and Bioscience, 3: 4.
https://doi.org/10.1186/s43170-021-00072-5
Marappan K., Sadasivam S., Natarajan N., Subramani M., Thangaraj M., and Arumugam V.A., 2026, Effect of indole-3-butyric acid and α-naphthaleneacetic acid on rooting of bottle brush [Callistemon lanceolatus (Sm.) Sweet] cuttings, Agricultural Science Digest, online first: 1-6.
https://doi.org/10.18805/ag.D-6485
Mataruga M., Cvjetković B., De Cuyper B., Aneva I., Zhelev P., Cudlín P., Metslaid M., Kankaanhuhta V., Collet C., Annighöfer P., Mathes T., Tsakaldimi M., Paitaridou D., Jónsdóttir R.J., Monteverdi M.C., de Dato G., Mariotti B., Kolevska D.D., Lazarević J., Fløistad I.S., Klisz M., Gil W., Paiva V., Fonseca T., Nicolescu V.N., Popović V., Devetaković J., Repáč I., Božič G., Kraigher H., Andivia E., Diez J.J., Böhlenius H., Löf M., Bilir N., and Villar-Salvador P., 2023, Monitoring and control of forest seedling quality in Europe, Forest Ecology and Management, 546: 121308.
https://doi.org/10.1016/j.foreco.2023.121308
Mello C.C., Rowe N., Soffiatti P., Zuffellato-Ribas K.C., and Sant’Anna-Santos B.F., 2025, Morphoanatomical aspects of stem cuttings of Selenicereus setaceus (Salm-Dyck) A. Berger ex Werderm. (Cactaceae), Brazilian Journal of Biology, 85: e293866.
https://doi.org/10.1590/1519-6984.293866
Mohammed A.A., Aziz R.R., Ahmad F.K., Noori I.M., and Ahmad T.A., 2020, Rooting capacity of hardwood cuttings of some fruit trees in relation to cutting pattern, Journal of the University of Duhok, 23(1): 1-6.
https://doi.org/10.26682/ajuod.2020.23.1.1
Morresi V., Capocasa F., Balducci F., Diamanti J., and Mezzetti B., 2025, Nursery propagation systems for high-quality strawberry (Fragaria × ananassa Duch.) plug plant production from micropropagated, soilless-grown mother plants, Horticulturae, 11(8): 888.
https://doi.org/10.3390/horticulturae11080888
Muniandi S.K., Ariff F.F.M., Harun S.T., Bahari S.N.S., Taini M.M., and Abdullah M.Z., 2025, Integrated propagation strategies for superior genotypes of Moringa oleifera L. to enhance sustainable planting material production, Forests, 16(12): 1863.
https://doi.org/10.3390/f16121863
Muniandi S.K., Ariff F.F.M., Pisar M., Harun S.T., Abdullah M.Z., Abdullah F., Hashim S.N.A.M., Bahari S.N.S., and Saffie N., 2024, Crop improvement of Moringa oleifera L. through genotype screening for the development of clonal propagation techniques of high-yielding clones in Malaysia, Biology, 13(10): 785.
https://doi.org/10.3390/biology13100785
Nión M., Ross S., González-Tálice J., Torres L., Bottarro S., Sotelo-Silveira M., Píriz-Pezzutto S., Antonelo F.A., and Fett-Neto A.G., 2026, Rooting ability of Eucalyptus dunnii Maiden mini-cuttings is conditioned by stock plant nighttime temperature, Plants, 15(2): 335.
https://doi.org/10.3390/plants15020335
Pandey A., Verma O., and Chand S., 2022, In vitro propagation of Alangium salviifolium (L. f.) Wangerin: an important tropical medicinal tree, Plant Cell, Tissue and Organ Culture, 148(1): 15-22.
https://doi.org/10.1007/s11240-021-02155-7
Pang J., Xiong Y., Zeng Y., Chen X., Li J., Zhang X., Li Y., Wu K., Zeng S., Teixeira da Silva J.A., and Ma G., 2024, Shoot organogenesis from Tetrastigma hemsleyanum leaf and petiole explants, and subsequent plant regeneration and acclimatization, Journal of Plant Growth Regulation, 43(12): 4782-4795.
https://doi.org/10.1007/s00344-024-11433-5
Pascual J.A., Ceglie F., Tuzel Y., Koller M., Koren A., Hitchings R., and Tittarelli F., 2018, Organic substrate for transplant production in organic nurseries, a review, Agronomy for Sustainable Development, 38(3): 35.
https://doi.org/10.1007/s13593-018-0508-4
Qahtan A.A., Faisal M., Alatar A.A., and Abdel-Salam E.M., 2021, High-frequency plant regeneration, genetic uniformity, and flow cytometric analysis of regenerants in Ruta chalepensis L., Plants, 10(12): 2820.
https://doi.org/10.3390/plants10122820
Quan J., Ni R., Wang Y., Sun J., Ma M., and Bi H., 2022, Effects of different growth regulators on the rooting of Catalpa bignonioides softwood cuttings, Life, 12(8): 1231.
https://doi.org/10.3390/life12081231
Rock R.R., An S., and Kim J., 2022, Optimum moisture conditions for English lavender cuttings are drier for root development than shoot development, Horticulturae, 8(8): 753.
https://doi.org/10.3390/horticulturae8080753
Saini P., Bishnoi A., Kathwal R., and Sharma R., 2025, Vegetative propagation techniques of fruit crops through cuttingsa review, International Journal of Farm Sciences, 15(4): 29-37.
https://doi.org/10.5958/2250-0499.2025.00054.8
Sarolia D.K., Meena R.K., Kumawat K.L., Choudhary M.K., and Singh D.K., 2021, Raising of quality saplings of arid horticultural crops: a review, Journal of Agriculture and Ecology, 11: 1-14.
https://doi.org/10.53911/jae.2021.11101
Savina O., Simochko V., Scheidyk K., Cvihun D., and Shakhnovych H., 2025, Evaluation of introduced hazelnut varieties for the ability to reproduce vegetatively, Plant Science (Horticulture, Agronomy, Viticulture), 5: 48-58.
https://doi.org/10.47279/Plantscience_2025-05-57
Schilisting T., Sá A.C.S., Da Silva Filho D.P., Da Silva V.M., Navroski M.C., De Oliveira Pereira M., Nascimento B., Moraes C., De Andrade R.S., Estopa R.A., and Miranda L., 2025, Developmental and physiological effects of the light source and cultivation environment on mini cuttings of Eucalyptus dunnii Maiden, Forests, 16(6): 901.
https://doi.org/10.3390/f16060901
Schrader H.K., Pessoa H.P., Enzenbacher T.B., Teh S.L., Anderson N.O., and Miller B.M., 2026, Asexual propagation of Salix humilis using stem cuttings I: cutting types, HortScience, 61(1): 48-55.
https://doi.org/10.21273/HORTSCI18991-25
Seleshi G., Firde K., Mosie T., and Setu H., 2021, Identification of cutting types for the successful regeneration of two plum (Prunus salicina Lindl) rootstock varieties, Advances in Life Science and Technology, 85: 19-24.
https://doi.org/10.7176/ALST/85-04
Seo J.M., Shin J.W., Park C.R., Kim Y.E., Lee J.W., Baek S.G., Kim J.M., Kim J.H., and Ahn C.H., 2023, Effect of propagation media and plant growth regulators on adventitious rooting of softwood cuttings of Apocynum lancifolium Russanov, Journal of People, Plants, and Environment, 26(6): 805-812.
https://doi.org/10.11628/ksppe.2023.26.6.805
Shen P., Wang L., Qureshi W.A., and Gao J., 2025, Influence of rhizosphere temperature and humidity regulation on rooting, mortality, and transplant survival of aeroponically rapid growth mulberry cutting, Agronomy, 15(3): 583.
https://doi.org/10.3390/agronomy15030583
Singh B., Rawat J.S., Gusain Y.S., Khanduri V.P., Riyal M.K., and Kumar P., 2021, Shoot position, cutting types and auxin treatments influence rooting response on Tecoma stans, Ornamental Horticulture, 27(2): 213-220.
https://doi.org/10.1590/2447-536x.v27i2.2262
Sun J., Li H., Chen H., Wang T., Quan J., and Bi H., 2023, The effect of hormone types, concentrations, and treatment times on the rooting traits of Morus ‘Yueshenda 10’ softwood cuttings, Life, 13(4): 1032.
https://doi.org/10.3390/life13041032
Ventura J.A., Lima I.M., Martins M.V.V., Culik M.P., and Costa H., 2019, Impact and management of diseases in the propagation of fruit plants, Revista Brasileira de Fruticultura, 41(4): e-647.
https://doi.org/10.1590/0100-29452019647
Vuong L.Q., Trinh D.T.X., Tham T.B., and Chau D.T.M., 2026, Optimization of the vegetative propagation protocol for Ardisia silvestris Pit. via stem cuttings in the Western Nghe An biosphere reserve, Vinh University Journal of Science, 55(1A): 116.
https://doi.org/10.56824/vujs.2025a0127a
Wang H., Wang A., Pu H., Yang Y., Ling Z., Xu H., Xu J., Yu H., and Wu X., 2023, Induction, flavonoids contents, and bioactivities analysis of hairy roots and true roots of Tetrastigma hemsleyanum Diels et Gilg, Molecules, 28(6): 2686.
https://doi.org/10.3390/molecules28062686
Wang L., Wang Q., Dong C., Teng C., Wang L., Zhou Y., Yang B., Kuang H., and Sun Y., 2025, Exploring Tetrastigma hemsleyanum polysaccharides: a recent advance in preparation, structural features, bioactivities, and potential application prospects, International Journal of Biological Macromolecules, 310: 143477.
https://doi.org/10.1016/j.ijbiomac.2025.143477
Wei K., Ruan L., Wang L., and Cheng H., 2019, Auxin-induced adventitious root formation in nodal cuttings of Camellia sinensis, International Journal of Molecular Sciences, 20(19): 4817.
https://doi.org/10.3390/ijms20194817
Xia J., Li X., Lin M., Yu J., Zeng Z., Ye F., Hu G., Miu Q., He Q., Zhang X., and Liang Z., 2023, Screening out biomarkers of Tetrastigma hemsleyanum for anti-cancer and anti-inflammatory based on spectrum-effect relationship coupled with UPLC-Q-TOF-MS, Molecules, 28(7): 3021.
https://doi.org/10.3390/molecules28073021
Xue G., Wu J., Zhou B., Zhu X., Zeng J., Ma Y., Wang Y., and Jia H., 2023, Effects of shading on the growth and photosynthetic fluorescence characteristics of Castanopsis hystrix seedlings of top community-building species in Southern Subtropical China, Forests, 14(8): 1659.
https://doi.org/10.3390/f14081659
Yang G.R., Jung H.H., Park K.Y., and Song K.J., 2022, Efficiency of closed cutting propagation affected by closed periods, leaflet number and photoperiod in rose (Rosa hybrida), Journal of Bio-Environment Control, 31(3): 212-220.
https://doi.org/10.12791/ksbec.2022.31.3.212
Yazar M., Genç H.E., Feyzioğlu F., Atar F., and Turna I., 2025, Effects of auxins, medium, and collection season on the rooting of Caucasian whortleberry (Vaccinium arctostaphylos L.) stem cuttings, Journal of Sustainable Forestry, 44(10): 931-948.
https://doi.org/10.1080/10549811.2025.2552717
Zhang M., Montanez C., Pearson B.J., Li Y., and Chen J., 2025, Aeroponics enables consistent cutting propagation of kratom (Mitragyna speciosa): impacts of photoperiod, cultivar, and rooting hormone, Frontiers in Plant Science, 16: 1650327.
https://doi.org/10.3389/fpls.2025.1650327
Zheng L., Xiao Z., and Song W., 2020, Effects of substrate and exogenous auxin on the adventitious rooting of Dianthus caryophyllus L., HortScience, 55(2): 170-173.
https://doi.org/10.21273/HORTSCI14334-19
Zheng T., Wei L., Xiang J., Zheng W., Wu J., and Cheng J., 2025, Optimal rooting substrates and hormonal regulation via a multi-omics analysis during Vitis davidii cutting rooting, Plant Stress, 16: 100851.
https://doi.org/10.1016/j.stress.2025.100851
Zhou F., Lu Y., Sun T., Sun L., Wang B., Lu J., Li Z., Zhu B., Huang S., and Ding Z., 2022, Antitumor effects of polysaccharides from Tetrastigma hemsleyanum Diels et Gilg via regulation of intestinal flora and enhancing immunomodulatory effects in vivo, Frontiers in Immunology, 13: 1009530.
https://doi.org/10.3389/fimmu.2022.1009530
Zhu R., Xu X., Ying J., Cao G., and Wu X., 2020, The phytochemistry, pharmacology, and quality control of Tetrastigma hemsleyanum Diels and Gilg in China: a review, Frontiers in Pharmacology, 11: 550497
https://doi.org/10.3389/fphar.2020.550497


. FPDF(win)
. FPDF(mac)
. HTML
. Online fPDF
Associated material
. Readers' comments
Other articles by authors
. Jianhui Li

Related articles
. Tetrastigma hemsleyanum
. Cutting propagation
. Adventitious root
. Standardized seedling production
. Seedling quality
Tools
. Post a comment