Research Insight
Effects of Potassium Fertilization on Fruit Size, Sugar Accumulation, and Quality of Citrus 

 Author Correspondence author
International Journal of Horticulture, 2026, Vol. 16, No. 4 doi: 10.5376/ijh.2026.16.0022
Received: 06 Jul., 2026 Accepted: 12 Aug., 2026 Published: 28 Aug., 2026
Zhang B., 2026, Effects of potassium fertilization on fruit size, sugar accumulation, and quality of citrus, International Journal of Horticulture, 16(4): 251-268 (doi: 10.5376/ijh.2026.16.0022)
With increasing consumer demand for high-quality citrus fruits, improving fruit size, sugar accumulation, and flavor attributes through nutritional regulation has become an important objective in orchard management. This study reviews the application of potassium fertilization in citrus production and summarizes recent advances in potassium uptake and transport, fruit growth, carbon metabolism regulation, and quality formation. The results indicate that appropriate potassium application can optimize nutrient allocation within citrus trees, promote the transport of photosynthetic assimilates to fruits, enhance fruit enlargement and sugar accumulation, and improve total soluble solids content and sugar–acid balance. However, citrus responses to potassium fertilization vary among cultivars, growing environments, and cultivation practices, while application timing, fertilization methods, and nutrient balance strongly influence management outcomes. Future integration of nutrient diagnosis, precision fertilization, and smart agriculture technologies may further improve potassium use efficiency and promote high-quality and sustainable citrus production.
1 Introduction
Citrus is one of the most economically important fruit crops worldwide, with major production and trade systems concentrated in countries such as China, Brazil, and the United States (Abouzari and Nezhad, 2016; Spreen et al., 2020; Wen et al., 2021). With increasing consumer demand for high-quality fresh fruit, improving and stabilizing citrus yield and fruit quality has become a major objective in modern orchard production. Fruit size, total soluble solids (TSS), sugar–acid ratio, and flavor-related traits directly influence consumer acceptance and market value (Wu et al., 2021; Morales Alfaro et al., 2023). However, citrus production still faces common challenges, including inconsistent fruit size, insufficient sugar accumulation, and a low proportion of premium-quality fruits. Therefore, optimizing nutrient management has become an important approach for improving citrus fruit quality.
Potassium (K) is one of the essential macronutrients required for plant growth and development and plays critical roles in carbon metabolism, photosynthesis, osmotic regulation, and assimilate transport (Hasanuzzaman et al., 2018; Johnson et al., 2022). Unlike nitrogen and phosphorus, which are mainly involved in structural components, potassium primarily regulates plant growth and yield formation through enzyme activation, stomatal movement, and source-sink relationships (Sardans and Peñuelas, 2021). In leaves, adequate potassium supply promotes photosynthetic carbon assimilation and enhances the transport of photosynthetic products to sink organs such as fruits. In contrast, potassium deficiency reduces photosynthetic capacity, restricts carbohydrate accumulation, and ultimately inhibits plant growth and yield formation (Tränkner et al., 2018; Shah et al., 2024). However, excessive potassium application may also reduce nutrient use efficiency and disturb the balance among mineral elements. Therefore, maintaining an appropriate potassium supply level is essential for improving crop production efficiency (Hasanuzzaman et al., 2018).
Citrus has a relatively high potassium demand, and large amounts of potassium accumulate during fruit development. Since potassium in citrus orchard soils is vulnerable to leaching losses, insufficient potassium supply often results in reduced fruit size, lower yield, and impaired fruit quality. Previous studies have demonstrated that appropriate potassium fertilization can promote fruit enlargement and enhance sugar accumulation. For example, Wu et al. (2024) reported that maintaining fruit potassium concentration at an appropriate level of approximately 1.5% in Newhall navel orange increased fruit growth rate, enhanced source–sink activity, and promoted sucrose transport from leaves to fruits, thereby improving fruit quality. In Cara Cara navel orange, potassium application at 0.50 kg per plant promoted the accumulation of sucrose, fructose, and glucose, which was closely associated with the regulation of sucrose metabolism-related enzyme activities (Wu et al., 2021). Foliar application of K2SO4 has also been shown to increase fruit weight, total soluble solids, soluble sugar content, and the TSS:TA ratio while reducing titratable acidity (Thu et al., 2024). Furthermore, Xu et al. (2024) found that optimized nutrient management in citrus orchards increased yield by 11.9%, single fruit weight by 2.8%, TSS by 5.9%, and total sugar content by 8.6%, indicating that balanced nutrient regulation plays an important role in improving fruit quality.
Although the importance of potassium in citrus quality formation has been widely recognized, the optimal potassium application rate, fertilizer type, and application timing remain variable under different production conditions. Citrus responses to potassium are influenced by multiple factors, including cultivar, rootstock, climatic conditions, and soil nutrient status. Moreover, excessive potassium input may lead to nutrient competition and inefficient resource utilization (Kuzin and Solovchenko, 2021; Sardans and Peñuelas, 2021). Therefore, clarifying the regulatory effects of potassium management on citrus fruit development and quality formation is important for improving fertilizer use efficiency and achieving high-quality and sustainable citrus production.
This study focuses on the effects of potassium fertilization on citrus fruit size, sugar accumulation, and quality formation, with particular emphasis on the roles of potassium in promoting fruit enlargement, regulating carbon assimilate transport, and improving sugar–acid balance. The aim is to clarify the relationship between potassium nutrition and citrus fruit quality development, thereby providing theoretical references for precision potassium management and the production of high-quality citrus fruits in modern orchards.
2 Physiological Functions of Potassium in Citrus Growth
2.1 Potassium uptake, transport, and distribution in citrus plants
Potassium in citrus is mainly absorbed by the root system and subsequently transported over long distances through the xylem and phloem to meet the physiological demands of metabolically active tissues (Wen et al., 2021; Wegner et al., 2025). Previous botanical studies have shown that after potassium is taken up from the soil, it is transported through the xylem to aboveground tissues along with the transpiration stream. Source tissues can then reload potassium into the phloem, allowing its redistribution to sink organs and partial recycling back to the root system (Dreyer et al., 2017). This recycling process has important physiological significance because potassium concentration gradients facilitate vascular transport processes, including sucrose reloading, while helping coordinate the balance between aboveground demand and root supply (Dreyer et al., 2017; Raddatz et al., 2020). Citrus plants also possess a relatively well-developed potassium transport system. Öz (2024) reported that 25 CsHAK genes have been identified in sweet orange (Citrus sinensis), and these HAK/KUP/KT transporter proteins are involved in potassium transport across the plasma membrane and within organelles.
Potassium is generally preferentially accumulated in organs with high metabolic activity, particularly leaves, where strong osmotic regulation and transport control are required. However, during citrus fruit development, fruits also function as important potassium sink organs (Sardans and Peñuelas, 2021; Jiao et al., 2022). In citrus orchards, the amount of potassium absorbed and exported by fruits is higher than that of other mineral nutrients, which explains why potassium deficiency can rapidly affect fruit quality and final yield in the current growing season.
Fertilization studies have further demonstrated that potassium supply can modify nutrient allocation patterns between vegetative organs and fruits. For example, Wen et al. (2021) showed that combined application of potassium fertilizer and organic fertilizer increased dry matter accumulation in spring flush leaves and shoots, while enhancing mineral nutrient uptake by both vegetative tissues and fruits. Root-zone potassium application also increased potassium, calcium, and nitrogen concentrations in citrus peel and pulp, indicating that external potassium supply can regulate internal nutrient distribution and promote greater nutrient transport toward developing fruit tissues (Figure 1) (Jiao et al., 2022).
|
Figure 1 Potassium uptake, transport, and source–sink regulation in citrus plants Image caption: The figure illustrates potassium uptake, transport, and source–sink regulation in citrus plants. Soil-derived K+ is absorbed by roots through HAK/KUP/KT transporters and transported upward via the xylem. In source leaves, potassium enhances stomatal regulation, photosynthesis, carbon assimilation, and sucrose synthesis. Subsequently, K+ facilitates phloem loading and assimilate transport toward fruit sink tissues, promoting potassium accumulation, sugar unloading, fruit enlargement, and quality improvement |
.png)
2.2 Potassium regulation of photosynthesis and carbon metabolism
Potassium directly regulates stomatal function and plant water relations, and sufficient potassium supply generally improves CO2 assimilation capacity and photosynthetic efficiency in citrus and other plant species (Wen et al., 2021; Johnson et al., 2022). Studies have shown that potassium fertilization increases the net photosynthetic rate, stomatal conductance, and intercellular CO2 concentration in citrus cultivars prone to fruit cracking, indicating that an adequate potassium level can improve leaf gas exchange processes (Jiao et al., 2022).
Broader studies across plant species have also demonstrated that potassium deficiency reduces photosynthetic carbon assimilation capacity, leading to impaired photosynthesis and decreased assimilate utilization efficiency (Anil Kumar et al., 2024). Physiologically, these effects are closely associated with the involvement of potassium in regulating membrane potential, intracellular pH stability, osmotic balance, and enzyme systems related to photosynthesis and respiration (Raddatz et al., 2020; Jiao et al., 2022).
Potassium promotes carbohydrate synthesis in source leaves and enhances the transport of photosynthetic products to fruits, thereby facilitating carbon metabolism in citrus plants (Wen et al., 2021). In Newhall navel orange, potassium application enhanced leaf photosynthesis, increased the activity of sucrose phosphate synthase (SPS) and the expression of the CsSPS gene, while also improving the activities of SPS and sucrose synthase (SS) in fruits, indicating that potassium simultaneously promotes metabolic processes in both source and sink tissues (Wu et al., 2024).
Further studies by Wu et al. (2024) demonstrated that potassium supply increased the accumulation of 13C-sucrose and 13C-glucose in fruits, suggesting that potassium enhances carbon transport from leaves to fruits during fruit enlargement and coloration stages. This transport effect has a clear physiological basis, as potassium is one of the major osmotic regulators in phloem sap and contributes to maintaining phloem pressure flow, thereby facilitating the transport of sucrose and other solutes (Tränkner et al., 2018).
2.3 Potassium and fruit development processes
Potassium promotes citrus fruit enlargement, partly because it regulates cellular osmotic potential and turgor pressure, both of which are fundamental processes underlying cell expansion (Wen et al., 2021; Wu et al., 2024). Jiao et al. (2022) demonstrated that potassium is associated with fruit cell division, root proliferation, and enhancement of peel tissues, suggesting that potassium not only affects fruit cell expansion but also contributes to maintaining the vegetative growth system that supports fruit development. At the whole-fruit developmental level, an adequate potassium supply can increase fruit growth rate in Newhall orange, while repeated foliar applications of K2SO4 during citrus development can also increase individual fruit weight (Wu et al., 2024). Related orchard studies further indicate that potassium promotes fruit enlargement, improves peel coloration, and alters peel thickness; however, these effects are influenced by potassium application rate, fertilizer type, and cultivation management practices (Wen et al., 2021).
Thu et al. (2024) reported that potassium enhances citrus fruit sink strength by coordinating sugar metabolism, transporter activity, and vascular transport of assimilates. In Newhall navel orange, maintaining fruit potassium concentration at an optimal level of approximately 1.5% improved fruit quality and promoted sugar accumulation (Wu et al., 2024). During citrus fruit development, foliar application of K2SO4 also increased soluble sugar content, total soluble solids (TSS), and the TSS:TA ratio, while upregulating the expression of genes associated with sugar metabolism and transport, including CsCWINV-2/6, CsSUT-1/2, and CsVPP-1/2. These findings further support the model that potassium promotes fruit quality formation by enhancing sink strength (Thu et al., 2024).
3 Effects of Potassium Fertilization on Citrus Fruit Size
3.1 Potassium effects on fruit growth and expansion
Previous studies have shown that potassium promotes fruit growth by enhancing cell division and cell elongation, while maintaining the turgor pressure required for cell expansion during fruit development (Toor et al., 2021; Jiao et al., 2022). In citrus, potassium promotes root proliferation and improves nutrient uptake capacity, thereby indirectly supporting rapid fruit growth during the cell division and enlargement stages (Jiao et al., 2022).
The timing of potassium supply is also critical, as citrus fruits exhibit different sensitivities to potassium availability throughout their developmental stages. Thu et al. (2024) found in Nanfeng mandarin that continuous foliar application of K2SO4 during the cell division, cell enlargement, and maturation stages produced greater growth-promoting effects than potassium application restricted to a single developmental stage. Studies on pomelo have also identified distinct periods of high potassium demand. Approximately two months after fruit set represents a critical developmental stage, indicating that potassium supply needs to coincide with peak fruit nutrient requirements to achieve optimal effects (Magbalot-Fernandez and Guzman, 2019).
Potassium fertilization generally increases fruit weight directly. In Kinnow mandarin, soil potassium application significantly increased individual fruit weight, fruit number, and overall yield (Singh et al., 2023). In Baladi lemon cultivated under potassium-deficient soil conditions, foliar potassium application improved fruit size-related traits. Among different treatments, potassium tartrate resulted in the highest individual fruit weight and volume in 2022, while high-concentration potassium citrate increased fruit weight, volume, and dry matter content across multiple seasons (Awad et al., 2024).
Magbalot-Fernandez and Guzman (2019) reported that increasing potassium application to 225 g per tree in ‘Magallanes’ pomelo increased individual fruit weight by 22%-26%, although fruit diameter and length did not show significant changes. This indicates that potassium can enhance fruit biomass accumulation but may not necessarily alter linear fruit size parameters. Studies on Newhall orange further confirmed the role of potassium in promoting fruit growth, showing that an adequate potassium level increased fruit growth rate and overall quality, with the optimal response occurring when fruit potassium concentration was maintained at approximately 1.5% (Wu et al., 2024).
3.2 Potassium regulation of source-sink relationships
One of the important pathways through which potassium promotes fruit enlargement is by improving leaf photosynthetic capacity and enhancing the supply capacity of source tissues. Studies have shown that potassium regulates stomatal movement, plant water relations, and photosynthetic processes (Hasanuzzaman et al., 2018; Johnson et al., 2022). For example, potassium deficiency in hydroponically grown lemon plants resulted in reductions in photosynthetic rate, stomatal conductance, transpiration rate, intercellular CO2 concentration, and pigment content, although different rootstock materials exhibited certain variations in their responses (Papadakis et al., 2023). In contrast, potassium application in citrus cultivars susceptible to fruit cracking increased photosynthetic rate, stomatal conductance, and intercellular CO2 concentration, indicating that adequate potassium supply improves leaf gas exchange capacity (Jiao et al., 2022). Foliar potassium application in lemon also increased SPAD values, photosynthetic performance index, and leaf nutritional status, which is consistent with the enhanced activity of source tissues under sufficient potassium availability (Awad et al., 2024).
Potassium can also promote fruit enlargement by enhancing carbohydrate transport from leaves to fruits. Wu et al. (2024) found in Newhall navel orange that potassium supply simultaneously enhanced both source strength and sink strength, increased fruit growth rate, and promoted sucrose transport from source leaves to fruits. Mechanistically, potassium enhances carbon transport through the symplastic loading pathway by increasing the number of plasmodesmata and the intensity of carboxyfluorescein signal transmission, indicating improved phloem loading capacity during fruit development.
Similar patterns have been observed in Cara Cara navel orange, where potassium increased sucrose, fructose, and glucose contents by regulating the activities of sucrose metabolism-related enzymes, thereby enhancing fruit sink strength (Wu et al., 2021). Studies on other non-citrus fruit trees have also demonstrated that potassium increases carbon import rates into sink organs and promotes the activity of enzymes involved in sugar conversion, which is consistent with the “source-sink regulation” model observed in citrus (Luo et al., 2021).
3.3 Factors influencing potassium responses in citrus
Citrus genotypes do not respond uniformly to potassium fertilization. A meta-analysis by Xu et al. (2024) demonstrated that different citrus groups, including mandarins, pomelos, and sweet oranges, showed distinct growth and yield responses after optimized fertilization. Specific experiments have further confirmed these differences. For example, potassium application in pomelo substantially increased fruit set, fruit number, and individual fruit weight, but had limited effects on fruit diameter and length (Magbalot-Fernandez and Guzman, 2019). In contrast, lemon plants showed strong selectivity toward potassium sources, with different potassium fertilizers (potassium citrate, potassium tartrate, and potassium nitrate) exhibiting advantages for different fruit quality parameters (Awad et al., 2024). Rootstock type also affects potassium utilization efficiency. Papadakis et al. (2023) reported that in lemon, the effects of potassium on plant growth, photosynthetic performance, and mineral nutrient distribution were regulated by rootstock genotype.
Environmental conditions also determine the effectiveness of potassium fertilization. Due to differences in soil properties and climatic conditions, citrus responses to potassium supply are not always consistent among orchard studies (Wen et al., 2021; Papadakis et al., 2023). Among environmental factors, water management is particularly important. In sweet orange production, fertigation with only 50% of the recommended nitrogen and potassium rates achieved the highest yield and increased nutrient use efficiency by 22%; however, applying 100% of the recommended fertilization rate did not provide additional benefits and may instead increase the risks of soil acidification and ammonium toxicity (Quaggio et al., 2019). Excessive potassium application may also cause nutrient imbalance. For example, in hydroponically grown lemon, high potassium concentrations reduced the overall uptake of phosphorus, calcium, magnesium, boron, manganese, and zinc, with these effects being particularly evident under the 6 mM potassium treatment (Papadakis et al., 2023).
Therefore, the positive effects of potassium fertilization on citrus fruit enlargement can only be achieved consistently when fertilizer rate, potassium source, application timing, cultivar characteristics, rootstock traits, and water availability are properly coordinated. Rational potassium management should be based on local production conditions and tree nutrient requirements, rather than simply increasing potassium input.
4 Effects of Potassium Fertilization on Sugar Accumulation
4.1 Potassium regulation of carbohydrate metabolism
Potassium regulates sucrose degradation during the early stage of citrus fruit development and sucrose resynthesis during the later stage, thereby affecting sugar accumulation in fruits. Wu et al. (2021) reported that potassium application in Cara Cara navel orange increased the cleavage activities of invertase and sucrose synthase (SS) during the early fruit development stage, promoting sucrose degradation into fructose and glucose. During the later ripening stage, potassium enhanced the synthesis direction activity of sucrose synthase and increased the activity of sucrose phosphate synthase (SPS), indicating that potassium promotes sucrose resynthesis during fruit maturation. This stage-dependent regulatory pattern is consistent with the general characteristics of citrus sugar metabolism, in which sucrose is the major storage sugar in citrus fruits. As a rate-limiting enzyme in sucrose biosynthesis, SPS generally shows increasing expression levels during fruit maturation and is positively correlated with sucrose accumulation (Lu et al., 2024). Studies on other fruit crops also provide supporting evidence, showing that potassium generally enhances SPS and SS activities, thereby promoting the accumulation of sucrose, glucose, and fructose and shifting carbon metabolism toward higher sugar accumulation (Zhang et al., 2018; Wang et al., 2024).
Potassium also promotes sugar accumulation by enhancing phloem loading, long-distance transport, and the capacity of fruits to absorb carbohydrates. In Newhall navel orange, 13C tracing analysis showed that potassium application increased 13C-sucrose accumulation in fruits during the enlargement stage and increased both 13C-sucrose and 13C-glucose contents during the coloration stage, demonstrating that potassium enhances carbon transport from source leaves to sink fruits (Wu et al., 2024). The study further indicated that approximately half of the sugars in citrus fruits originate from transported carbohydrates, and potassium strengthens carbon flow between source and sink tissues by regulating the symplastic loading pathway.
In Nanfeng mandarin, continuous foliar application of K2SO4 throughout fruit development increased soluble sugar content, mainly due to enhanced fruit sink strength and sugar transport capacity induced by potassium (Thu et al., 2024). This transport-centered regulatory model is also supported by broader studies in plant nutritional physiology, which demonstrate that potassium is closely associated with the translocation of photosynthetic products from source leaves to sink fruits (Shah et al., 2024; 2025).
4.2 Molecular mechanisms of potassium-induced sugar accumulation
One of the important molecular mechanisms by which potassium promotes sugar accumulation is through enhancing the expression of sugar transport-related genes in leaves and fruits. In Nanfeng mandarin, foliar application of K2SO4 increased the expression of CsCWINV-2/6 in the segment membrane tissues and enhanced the expression of CsSUT-1/2 and CsVPP-1/2 in juice sac tissues, linking potassium nutrition with stronger fruit sink activity and sucrose unloading processes (Thu et al., 2024). In Newhall navel orange, potassium enhanced symplastic loading capacity, increased carboxyfluorescein signal intensity, and promoted plasmodesmata density in leaves, indicating that potassium not only affects the expression of sugar transport proteins but also modifies the structural pathways involved in carbohydrate transport (Wu et al., 2024). Sugar storage in citrus fruits also depends on vacuolar transport capacity. A proteomic study by Mao et al. (2024) revealed that tonoplast transporters such as TMT2 and STP7 may participate in regulating sugar accumulation within citrus fruit vacuoles. Related studies in tomato, melon, and magnesium-treated citrus have also demonstrated similar regulatory patterns, showing that potassium or other nutritional treatments can increase the expression of SUT, SWEET, VPP, and vacuolar sugar transporter genes, thereby enhancing sugar import and storage capacity in fruits (Wu et al., 2023; Han et al., 2024; Shah et al., 2025).
Potassium-induced sugar accumulation does not rely solely on sugar transport processes but also involves regulation of carbon metabolism-related gene networks. In Newhall navel orange, potassium increased the activities of key sucrose metabolism enzymes and the expression of related genes in both fruits and leaves, indicating that potassium coordinates carbon metabolism in source tissues with sugar utilization in sink tissues (Wu et al., 2024). Citrus SPS genes themselves are regulated by multiple factors, including developmental stage, tissue type, light conditions, hormone levels, and abiotic stresses, suggesting that external nutritional signals, such as potassium, may be integrated into broader sugar signaling regulatory networks (Lu et al., 2024). Further co-expression analysis revealed that WRKY transcription factors, particularly CsWRKY20, may participate in regulating citrus sugar accumulation through the CsSPS-mediated pathway. Studies in grapevine and melon also support this integrated regulatory model, showing that potassium-responsive genes are mainly enriched in pathways related to carbon metabolism, glycolysis/gluconeogenesis, fructose and mannose metabolism, as well as SPS/SUS-mediated regulation (Wang et al., 2024; Shah et al., 2025).
4.3 Relationship between potassium supply and soluble solids content
Adequate potassium supply generally results in a stable increase in total soluble solids (TSS) and soluble sugar content in citrus fruits. In Nanfeng mandarin, six consecutive foliar applications of K2SO4 significantly increased fruit TSS and soluble sugar content (Thu et al., 2024). In Cara Cara navel orange, potassium application increased sucrose, fructose, and glucose contents, as well as the ratio of total soluble sugars to citric acid, with the most pronounced improvement observed at an application rate of 0.50 kg potassium per tree (Wu et al., 2021). A meta-analysis conducted by Xu et al. (2024) on Chinese citrus production systems also demonstrated that optimized fertilization management increased TSS by 5.9% and total sugar content by 8.6%. Studies on other fruit crops have shown similar dose–response patterns, indicating that moderate potassium supply generally improves TSS and sugar accumulation more consistently than excessive potassium application (Zhang et al., 2018; Wang et al., 2024).
The effects of potassium on citrus flavor quality are not limited to sugar accumulation but also involve regulation of sugar–acid balance. In Cara Cara navel orange, potassium increased citric acid content by enhancing the activities of citrate synthase and phosphoenolpyruvate carboxylase, while simultaneously increasing the ratio of total soluble sugars to citric acid, thereby improving overall flavor balance (Wu et al., 2021). In contrast, in Nanfeng mandarin, foliar application of K2SO4 reduced titratable acidity and increased the TSS:TA ratio, indicating that the effects of potassium on organic acid metabolism are influenced by cultivar characteristics and application strategies (Thu et al., 2024).
Broader integrated studies on citrus have shown that optimized fertilization can reduce titratable acid (TA) and total acid contents while increasing the TSS/TA and TSC/TAC ratios, thereby improving overall fruit quality (Xu et al., 2024). This variation in acidity responses is also consistent with findings from non-citrus crops, where potassium may either promote citric acid synthesis or reduce malic acid and total acid accumulation, depending on plant species, developmental stage, and fertilizer source (Zhang et al., 2018; Wu et al., 2023).
5 Effects of Potassium Fertilization on Citrus Fruit Quality
5.1 Influence on external quality characteristics
Potassium improves the external quality of citrus fruits mainly by promoting fruit enlargement, enhancing peel coloration, and improving market appearance. In Newhall navel orange, combined application of potassium fertilizer and organic fertilizer improved fruit surface color and reduced peel thickness, resulting in a more desirable appearance for consumers (Wen et al., 2021). Shrestha et al. (2025) found that in HLB-tolerant Sugar Belle citrus grown under sandy soil conditions, foliar potassium application improved peel color and overall fruit quality; potassium nitrate applied in July or from May to July increased fruit size to more than 65 mm. In Page mandarin, potassium-containing foliar nutrient treatments increased fruit diameter and improved peel color parameters, including L*, a*, and b* values, which were consistent with enhanced visual quality (ValizadehKaji and Mohammaei, 2025). In Fremont mandarin, potassium nitrate application promoted fruit enlargement and improved fruit color and appearance, although most internal quality parameters showed limited changes in this experiment (Ülker and Kamiloğlu, 2021).
Potassium also influences peel development and firmness, both of which are important for fruit transportation performance and resistance to physiological disorders. Jiao et al. (2022) reported that potassium application in a citrus hybrid susceptible to fruit cracking increased the ratio of peel firmness to pulp firmness, enhanced potassium, calcium, and nitrogen accumulation in both peel and pulp tissues, and alleviated fruit cracking. The same study system and related citrus research indicate that sufficient potassium supply promotes peel tissue development and structural strengthening, thereby reducing the risk of fruit cracking (Jiao et al., 2022; Shrestha et al., 2025). In Sugar Belle citrus, foliar potassium application before autumn increased peel thickness to approximately 1.15 times that of the control, while combined potassium and boron application improved peel puncture resistance (Shrestha et al., 2025). In sweet lime, foliar application of KNO3 increased fruit firmness and juice content, which is consistent with the role of potassium in maintaining cell membrane stability and regulating vacuolar osmotic balance (Khan et al., 2025).
However, the effects of potassium on fruit quality are not always consistent. In ‘Salustiana’ orange, high potassium supply reduced magnesium and calcium accumulation in the flavedo but did not significantly alter peel thickness, external color, firmness, total soluble solids content, or acidity (Manzi et al., 2026).
5.2 Influence on internal quality traits
The most consistent effects of potassium on improving citrus internal quality are mainly reflected in increased total soluble solids (TSS), enhanced soluble sugar accumulation, and improved sugar–acid balance. In Newhall navel orange, an appropriate fruit potassium concentration (approximately 1.5%) promoted sugar accumulation and improved fruit quality, with both field and pot experiments directly demonstrating increased TSS after potassium application (Wu et al., 2024). In Valencia orange, the application of 0.5 kg nitrogen fertilizer and 0.9 kg potassium fertilizer per tree resulted in the highest TSS and TSS/TA ratio, whereas increasing potassium application rates further tended to increase juice acidity (Nguyen and Tai, 2020).
A meta-analysis of 92 studies conducted by Xu et al. (2024) showed that optimized fertilization with an appropriate increase in K2O input increased fruit TSS by 5.9%, total sugar content by 8.6%, reduced total acidity by 3.4%, and increased the TSS/TA ratio by 14.0%. However, it should be noted that excessive potassium application may negatively affect internal fruit quality in some production systems by increasing acidity and reducing the sugar–acid ratio (Shrestha et al., 2025).
Studies have shown that potassium can improve vitamin C content and influence secondary metabolic processes, although these responses are more complex than changes in TSS. In Newhall orange, combined application of potassium fertilizer and organic fertilizer not only increased TSS and the sugar–acid ratio but also promoted vitamin C accumulation (Wen et al., 2021). In sweet lime, lower concentrations of KNO3 increased vitamin C content, which may be related to the regulatory effects of potassium on sugar metabolism and ascorbic acid biosynthesis (Khan et al., 2025).
Potassium also alters metabolite composition in citrus peel and pulp, enhancing amino acid biosynthesis in peel tissues and glycoside accumulation in pulp tissues. Jiao et al. (2022) used the fruit-cracking-susceptible citrus hybrid ‘Ehime Kashi No. 34’ as the experimental material and evaluated three potassium levels. The results showed that potassium treatments increased K, N, and Ca concentrations in both peel and pulp, while improving the peel-to-pulp firmness ratio, photosynthetic rate, and stomatal conductance. Metabolomic analysis identified 59 and 13 differential metabolites in peel and pulp tissues, respectively. Changes in peel metabolism were mainly associated with enhanced amino acid biosynthesis, whereas pulp tissues showed increased accumulation of glycoside-related metabolites. The study suggested that potassium alleviates fruit cracking by coordinating peel mechanical strength with metabolic changes in internal and external tissues, thereby reducing the imbalance between pulp expansion and peel extension during fruit development.
5.3 Potassium optimization for different citrus quality targets
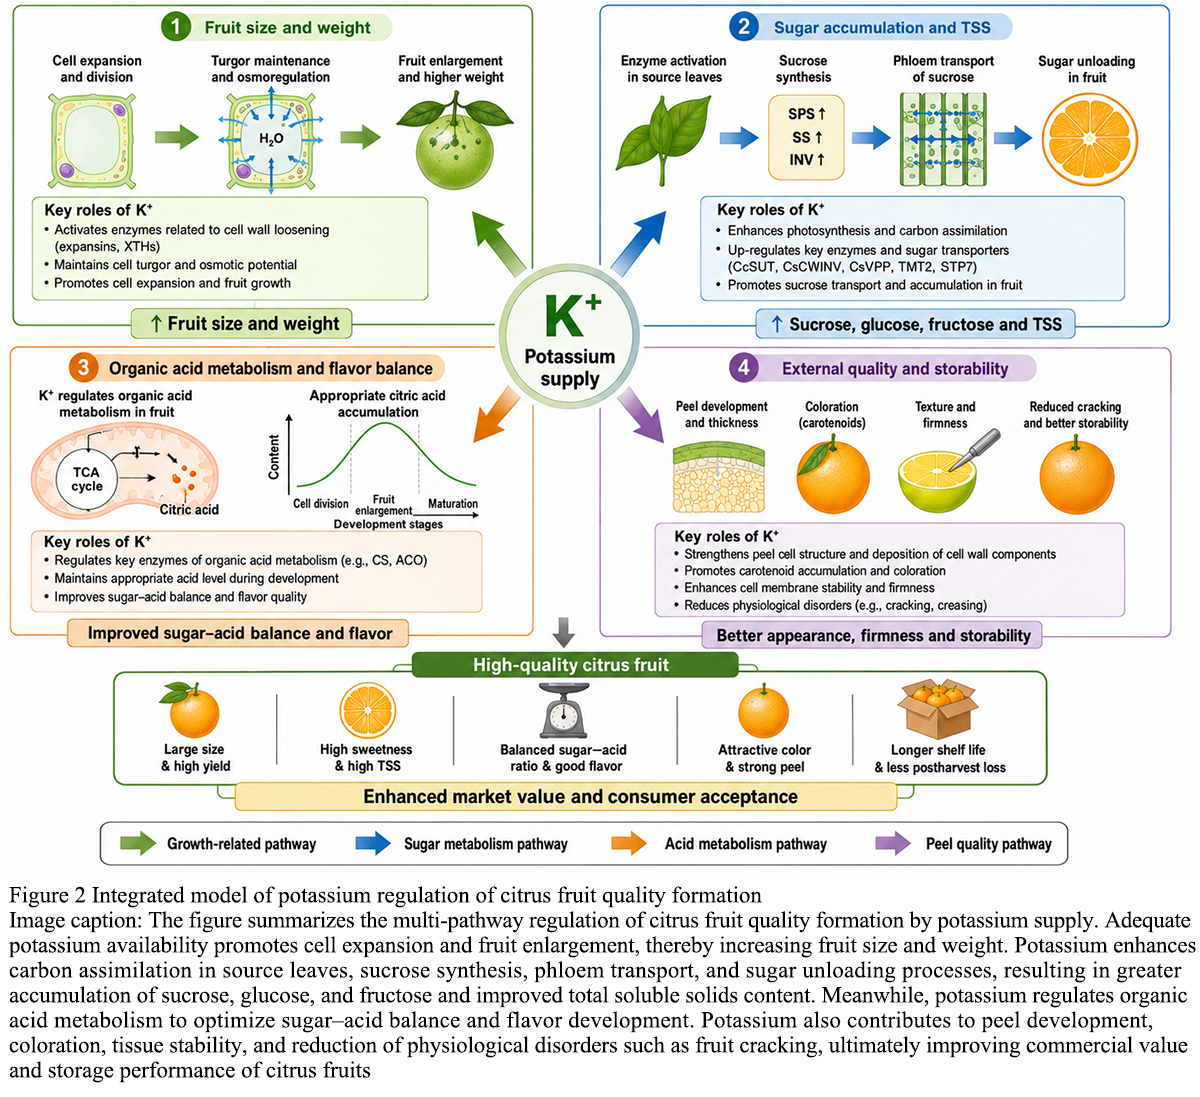
Potassium regulates citrus quality formation mainly through the coordinated regulation of multiple processes, including fruit growth, carbohydrate metabolism, organic acid balance, and peel development (Figure 2). For high-sugar citrus production, current evidence supports an appropriate and timely potassium supply rather than pursuing the maximum potassium application rate. For example, Chen et al. (2026) reported that in semi-arid regions of southwestern China, increasing fertilizer input during stage III enhanced soluble sugar and vitamin C accumulation, while reducing irrigation and increasing fertilizer levels during stage IV also promoted the accumulation of sugars and vitamin C. Since commercial citrus maturity largely depends on the ratio of soluble solids to acidity and juice percentage, potassium management aimed at improving sweetness should consider both cultivar characteristics and environmental conditions (Lado et al., 2018; Jiao et al., 2023).
|
Figure 2 Integrated model of potassium regulation of citrus fruit quality formation Image caption: The figure summarizes the multi-pathway regulation of citrus fruit quality formation by potassium supply. Adequate potassium availability promotes cell expansion and fruit enlargement, thereby increasing fruit size and weight. Potassium enhances carbon assimilation in source leaves, sucrose synthesis, phloem transport, and sugar unloading processes, resulting in greater accumulation of sucrose, glucose, and fructose and improved total soluble solids content. Meanwhile, potassium regulates organic acid metabolism to optimize sugar-acid balance and flavor development. Potassium also contributes to peel development, coloration, tissue stability, and reduction of physiological disorders such as fruit cracking, ultimately improving commercial value and storage performance of citrus fruits |
6 Potassium Fertilization Strategies in Citrus Orchards
6.1 Timing and methods of potassium application
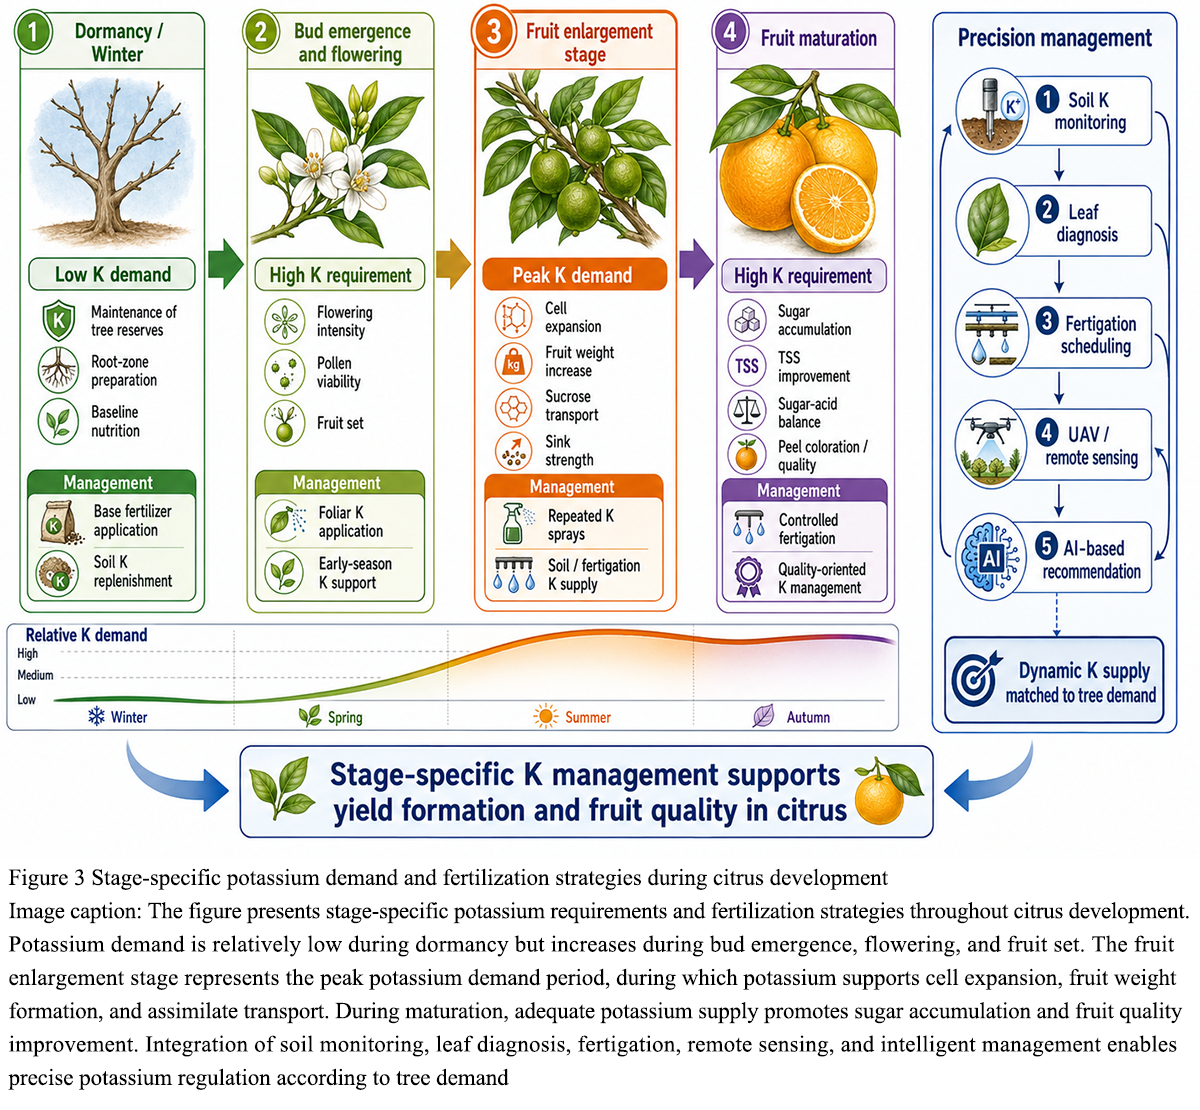
Potassium demand in fruit trees changes throughout different phenological stages, with the highest requirement generally occurring during rapid fruit growth and ripening stages. In citrus production, field studies have similarly demonstrated that flowering and fruit enlargement periods are critical stages for potassium management (Figure 3). Khan and Nabi (2023) used 20-year-old sweet lime (Citrus limetta) trees to compare the effects of foliar applications of KCl, K2SO4, and KNO3 on different application dates, including February 15, February 25, March 7, and March 17. The results showed that potassium application on March 17, 13 days after bud emergence, produced the best performance, with an average of 739.52 fruits per tree and a yield of 63.68 kg per tree, while reducing the time required for full bloom to 20 days. Among different potassium sources, the KNO3 treatment resulted in 808.75 fruits per tree, a yield of 69.48 kg per tree, and an average fruit weight of 85.64 g. The study indicated that potassium application after bud emergence in spring was more effective than application during the late winter dormancy period, suggesting that the period from spring bud development to flowering represents a critical window influencing flowering progression, fruit number, and yield formation.
|
Figure 3 Stage-specific potassium demand and fertilization strategies during citrus development Image caption: The figure presents stage-specific potassium requirements and fertilization strategies throughout citrus development. Potassium demand is relatively low during dormancy but increases during bud emergence, flowering, and fruit set. The fruit enlargement stage represents the peak potassium demand period, during which potassium supports cell expansion, fruit weight formation, and assimilate transport. During maturation, adequate potassium supply promotes sugar accumulation and fruit quality improvement. Integration of soil monitoring, leaf diagnosis, fertigation, remote sensing, and intelligent management enables precise potassium regulation according to tree demand |
In sweet orange, two to three foliar sprays applied around late April, May, and August improved yield and fruit size, with 4% KNO3 showing the best performance among the tested foliar fertilization treatments. In Washington navel orange, five foliar potassium applications from March to July improved leaf nutrient status, yield, and fruit quality, indicating that a staged potassium supply strategy during early reproductive growth and fruit development can provide positive effects (Al-Sabbagh and El-Gioushy, 2024).
Soil potassium application remains the primary potassium management strategy in orchards because it can continuously support root uptake throughout the growing season. However, citrus studies have shown that foliar potassium application plays an important complementary role when soil conditions limit nutrient availability. Ahmad et al. (2022) reported that in alkaline or calcareous citrus soils, soil fertilization alone often fails to achieve optimal leaf nutrient levels, making foliar fertilization an effective rapid correction method. Field comparisons in citrus have demonstrated that both basal soil potassium application and foliar potassium spraying promote plant growth and improve fruit quality. However, foliar application generally produces faster or more pronounced quality responses, whereas soil potassium application is more effective for increasing fruit weight and maintaining long-term tree nutrient supply (Tahir et al., 2023).
Fertigation provides a more precise approach for potassium management by matching potassium supply with seasonal nutrient requirements and root-zone environmental conditions. Based on lysimeter experiments in citrus, Zayani et al. (2024) found that nutrient concentrations in soil solutions varied substantially with irrigation amount, fertilizer input, and soil conditions, indicating that data-driven fertigation management based on real-time monitoring has advantages over fixed fertilization schedules.
6.2 Optimization of potassium application rates and nutrient balance
When potassium deficiency occurs in citrus orchards, increasing potassium supply generally improves plant performance. However, this response is not always linear, and excessive potassium application may reduce fertilizer use efficiency or cause nutrient imbalances. A meta-analysis of 92 citrus fertilization studies conducted by Xu et al. (2024) showed that optimized fertilization strategies increased K2O application by an average of 6.6% compared with conventional fertilization practices, while simultaneously improving fertilizer productivity, yield, individual fruit weight, total soluble solids content, sugar content, and the sugar–acid ratio. The greatest production benefits were mainly achieved through integrated nutrient management, particularly strategies involving optimized N-P-K ratios combined with the application of secondary and micronutrients.
Experiments with different potassium application rates have also supported this pattern. In ‘Salustiana’ orange, low, medium, and high annual potassium application rates altered potassium concentrations in leaves and flavedo tissues, but high potassium supply did not further improve the measured fruit quality parameters (Manzi et al., 2026). In Newhall navel orange, moderate application of organic fertilizer combined with potassium sulfate produced the best fruit quality performance, with a recommended K2SO4 application rate of 1.15-1.20 kg per tree under the tested soil conditions (Wen et al., 2021).
For a long time, citrus nutrient management recommendations have suggested that potassium supply should be maintained at a level close to nitrogen supply to achieve high yield and superior fruit quality (Khan and Nabi, 2023). However, excessive potassium availability may inhibit calcium and magnesium uptake. In hydroponically grown lemon, high potassium concentrations reduced the overall uptake of phosphorus, calcium, magnesium, boron, manganese, and zinc, with these effects being particularly evident at 6 mM potassium concentration (Papadakis et al., 2023). Brital et al. (2024) further found in Valencia orange orchards in Morocco that potassium-magnesium antagonism could still occur in leaves even when soil potassium availability was sufficient, indicating that soil potassium content alone cannot accurately reflect the nutritional balance status of citrus trees.
6.3 Precision potassium management
In recent years, commercial orchard data analysis has provided more quantitative evidence for potassium management. For example, Lima Neto et al. (2025) used boundary line analysis to estimate the optimal soil potassium concentration range for citrus orchards as 161.4-326.0 mg/dm3 and the suitable leaf potassium concentration range as 7.8-11.3 g/kg. The study also established optimal ranges for other nutrients, including nitrogen, calcium, and magnesium. Monitoring studies in Clementine mandarin orchards in Morocco similarly revealed substantial variations in soil solution nutrient availability and leaf nutrient composition among different fields and phenological stages, highlighting the importance of continuous leaf nutrient diagnosis (Zayani et al., 2024).
Precision potassium management is increasingly moving toward data-driven approaches. For example, unmanned aerial vehicle (UAV)-based multispectral imaging combined with machine learning techniques can accurately estimate major nutrient concentrations, including potassium, in citrus trees and generate spatial nutrient distribution maps for commercial orchards, providing a basis for site-specific fertilization management (Costa et al., 2022). More broadly, intelligent fertilizer recommendation systems integrating artificial intelligence (AI), the Internet of Things (IoT), and interpretable models demonstrate that real-time soil and climate data can support more accurate and explainable fertilization decisions (Venkateswara and Padmanaban, 2025). Studies in other fruit crops have also confirmed the practical value of adjusting potassium fertigation programs according to actual crop load and using machine vision technologies to optimize potassium demand prediction. These approaches may provide useful references for citrus orchards, where fruit load often varies considerably among different production years (Kuzin et al., 2020).
7 Integrated Potassium Management for Citrus Orchards
7.1 Coordination of potassium with other nutrient management
Potassium management should be considered as a component of an integrated nutrient management system because fruit growth and quality formation depend more on the coordinated uptake of nitrogen, phosphorus, and potassium rather than potassium supply alone. Ma et al. (2022) reported that drip fertigation improved fruit total soluble solids (TSS), titratable acidity (TA), and vitamin C content while increasing nitrogen, phosphorus, and potassium accumulation in fruits. The underlying mechanism was mainly attributed to nitrogen promoting sugar synthesis through enhanced photosynthesis, whereas phosphorus and potassium contributed more directly to sugar accumulation and regulation of the sugar-acid ratio. Field monitoring in Clementine mandarin orchards in Morocco similarly showed that optimized fertilization programs required increased nitrogen and potassium inputs compared with conventional local practices; however, monthly leaf nutrient diagnosis indicated that the major limitation was not simply insufficient annual nutrient supply but rather an inappropriate temporal distribution of nitrogen and potassium availability (Zayani et al., 2024). In Washington navel orange, repeated foliar applications of KNO3 improved leaf nutritional status, productivity, and fruit quality, suggesting that potassium can be combined with nitrogen through a single fertilizer source during periods of high canopy nutrient demand (Al-Sabbagh and El-Gioushy, 2024).
Interactions among potassium, calcium, and magnesium are also highly important, as the balance of cation supply influences peel integrity, root health, and fruit development. For example, in a citrus hybrid susceptible to fruit cracking, potassium application increased calcium, nitrogen, and potassium concentrations in both peel and pulp tissues and improved the peel-to-pulp firmness ratio, which was associated with reduced fruit cracking incidence (Jiao et al., 2022). A field-scale analysis of fruit cracking in Bingtang sweet orange by Shi et al. (2025) further demonstrated that soil calcium, potassium, and magnesium were important factors affecting cracking severity. Fruit cracking rate was negatively correlated with soil calcium and potassium concentrations but positively correlated with soil magnesium content.
However, excessive potassium supply may aggravate cation imbalance. In ‘Salustiana’ orange, high potassium treatments increased potassium accumulation in leaves and flavedo tissues but reduced calcium and magnesium accumulation in fruit tissues (Stagno et al., 2024). Such nutrient imbalance is relatively common in commercial production. A survey in southwestern China found that severe magnesium deficiency was closely associated with excessive nitrogen and potassium fertilization. Optimized management practices involving magnesium supplementation and reduced N-P-K inputs improved yield, fruit quality, nutrient use efficiency, and economic returns (Wang et al., 2022).
7.2 Integration of potassium fertilization with irrigation management
Potassium use efficiency is highly dependent on soil water conditions. In citrus orchards, potassium is prone to leaching losses, while water deficits and irregular rainfall patterns can alter potassium uptake processes and influence the occurrence of physiological disorders in fruits. A two-year citrus field experiment showed that maintaining 70% soil moisture combined with alginate oligosaccharide application increased yield by 11.93%-13.31%, total soluble sugar content by 15.16%-17.47%, sucrose content by 18.92%-20.81%, fruit potassium concentration by 51.09%-62.21%, and water use efficiency by 12.01%-13.34%. This treatment performed better than both higher and lower irrigation regimes (Li et al., 2024). The same treatment also enhanced net photosynthetic rate and root growth, increased available potassium content in the 0-20 cm soil layer, and reduced potassium movement into deeper soil layers, indicating that suitable soil moisture conditions improve potassium retention in soil and enhance plant potassium utilization.
Similar conclusions were reported by Stagno et al. (2024) in a deficit irrigation study on orange trees. Water-saving irrigation strategies reduced irrigation volume by 25%-49% without reducing yield, while improving water use efficiency and maintaining generally adequate mineral nutrition levels. However, leaf potassium concentrations under these treatments were often below the recommended range. These irrigation regimes also increased fruit vitamin C content, pulp coloration, and sugar concentration, suggesting that moderate water regulation can work synergistically with potassium management to improve fruit quality.
In citrus production, drip fertigation improves fruit TSS and juice percentage, enhances nitrogen, phosphorus, and potassium uptake, and reduces nitrogen and potassium losses through leaching and runoff compared with conventional fertilizer application methods such as broadcasting, hole application, or irrigation-based fertilizer delivery. Ma et al. (2022) found that drip fertigation could still promote citrus growth and development even with a 60% reduction in fertilizer input, indicating substantial potential for improving potassium use efficiency while reducing total fertilizer consumption. Monitoring results from mobile lysimeters in Moroccan citrus orchards further demonstrated that nutrient concentrations in soil solutions fluctuate significantly with irrigation amount, fertilizer input, and soil conditions. Therefore, water and fertilizer management based on real-time monitoring is more effective than fixed fertilization schedules (Zayani et al., 2024).
7.3 Application of precision potassium management in citrus orchards
Precision potassium management requires integration of soil testing and leaf nutrient diagnosis. Ahmad et al. (2022) conducted field investigations in calcareous citrus soils and found that soil potassium concentrations at different soil depths were generally at moderate levels, while deficiencies of nitrogen and micronutrients in leaves were widespread. This indicated that soil fertilization alone may not fully satisfy tree nutrient requirements, and foliar fertilization should be incorporated to improve orchard nutritional status. In recent years, boundary line analysis based on commercial orchard data has provided more accurate reference ranges. The study estimated that suitable potassium concentrations for citrus orchards were 161.4-326.0 mg/dm3 in soil and 7.8-11.3 g/kg in leaves, which can serve as practical guidelines for precision potassium fertilization recommendations (Lima Neto et al., 2025).
Precision fertilization strategies also need to be adjusted according to cultivar characteristics and developmental stages. In Clementine mandarin orchards, the fertilization requirements of the cultivars ‘Nour’, ‘Orogrande’, and ‘Nules’ differed, and monthly leaf nutrient diagnosis indicated that potassium should be supplemented in a timely manner before and during fruit growth and ripening stages (Zayani et al., 2024). In ‘Magallanes’ pomelo, key growth periods were mainly concentrated in May and August, while April represented the peak period for flowering and fruit set. The two months after fruit set were identified as a critical developmental stage, suggesting that potassium supply should be synchronized with these key physiological periods (Magbalot-Fernandez and Guzman, 2019). This study further showed that potassium application rates recommended based on soil analysis promoted canopy growth, whereas higher potassium inputs further increased flowering intensity, fruit set, fruit number, individual fruit weight, and yield, indicating that the optimal potassium rate depends on specific production objectives.
Studies on lemon and Kinnow mandarin further demonstrate that fertilization methods and treatment combinations should be matched with production goals. Foliar application of NG-K was more effective than basal application of sulfate of potash (SOP) in improving sugar accumulation and juice quality parameters (Tahir et al., 2023). Among different management strategies, application of a salicylic acid (SA) + potassium (K) + zinc (Zn) combination across three growth stages showed the most consistent effects in reducing fruit drop and improving juice quality across multiple locations (Anwar et al., 2022).
8 Advances and Future Trends in Citrus Potassium Management
Potassium is an essential nutrient that influences citrus tree growth and fruit quality formation, playing important roles in photosynthetic carbon assimilation, assimilate transport, fruit development, and quality regulation during maturation. Current studies indicate that appropriate potassium supply can improve leaf photosynthetic capacity, enhance material transport between source and sink tissues, and promote fruit enlargement and sugar accumulation. The effectiveness of potassium management is affected by multiple factors, including cultivar characteristics, rootstock type, soil conditions, water availability, and fertilization practices. Developing potassium management strategies adapted to different production conditions is therefore an important basis for achieving high-quality and efficient citrus production.
The regulatory effects of potassium on citrus fruit development are mainly associated with improved cellular expansion conditions, enhanced fruit growth, and strengthened nutrient supply capacity of the tree. Potassium demand is generally higher during rapid fruit growth and maturation stages, and timely potassium supplementation can improve fruit weight and marketability. Different citrus groups show distinct responses to potassium supply, with some cultivars exhibiting stronger effects on fruit enlargement, whereas others respond more significantly in terms of sugar accumulation and flavor improvement. In practical production, fertilization strategies should be adjusted according to cultivar characteristics and developmental stages to improve the synchronization between potassium supply and tree nutrient requirements.
The role of potassium in fruit quality formation is closely related to carbon metabolism and sugar transport processes. An appropriate potassium level promotes the translocation of photosynthetic products to fruits, regulates the activities of sucrose metabolism-related enzymes, and affects sugar transport processes, ultimately improving total soluble solids content and sugar–acid balance. However, excessive potassium supply may interfere with the uptake of calcium, magnesium, and other mineral elements, resulting in nutrient imbalance and reduced fertilizer use efficiency. Therefore, maintaining a balanced relationship between potassium and other mineral nutrients is essential for producing high-quality citrus fruits, and excessive potassium input should be avoided.
Future research should further improve precision potassium management systems in citrus orchards. Potassium requirements under different cultivar–rootstock combinations and ecological regions need to be validated through long-term field experiments, combined with leaf nutrient diagnosis and soil nutrient monitoring to establish more reliable evaluation indicators. The molecular basis underlying potassium regulation of fruit quality formation also requires further investigation, particularly regarding the interactions between potassium signaling, sugar metabolism networks, hormonal regulation, and fruit ripening processes.
With the development of fertigation, remote sensing, and smart agriculture technologies, citrus potassium management is expected to become increasingly dynamic and precise. Integrating soil, plant, and environmental information for nutrient demand prediction can improve potassium use efficiency and reduce resource losses. Future studies should strengthen the coordination of potassium management with irrigation, nitrogen and phosphorus nutrition, and micronutrient regulation, aiming to establish a more efficient, stable, and sustainable citrus nutrient management system and provide theoretical support and technical guidance for the development of modern citrus production.
Acknowledgments
The authors would like to express their sincere gratitude to Mr. Li for his assistance in organizing the literature materials. The authors also extend special thanks to the two anonymous peer reviewers for their comprehensive evaluation of the manuscript.
Conflict of Interest Disclosure
The authors affirm that this research was conducted without any commercial or financial relationships that could be construed as a potential conflict of interest.
Abouzari A., and Nezhad N.M., 2016, The investigation of citrus fruit quality, popular characteristic and breeding, Acta Universitatis Agriculturae et Silviculturae Mendelianae Brunensis, 64(3): 725-740.
https://doi.org/10.11118/actaun201664030725
Ahmad N., Hussain S., Ali M., Minhas A., Waheed W., Danish S., Fahad S., Ghafoor U., Baig K.S., Sultan H., Hussain M., Ansari M.J., Marfo T.D., and Datta R., 2022, Correlation of soil characteristics and citrus leaf nutrients contents in current scenario of Layyah District, Horticulturae, 8(1): 61.
https://doi.org/10.3390/horticulturae8010061
Al-Sabbagh M.N., and El-Gioushy S.F., 2024, Effects of different potassium forms on the nutritional status, productivity, and fruit quality of Washington navel orange trees, Annals of Agricultural Science, Moshtohor, 62(1): 115-128.
https://doi.org/10.21608/assjm.2024.294690.1290
Anil Kumar S., Kaniganti S., Hima Kumari P., Sudhakar Reddy P., Suravajhala P., P S., and Kishor P.K., 2024, Functional and biotechnological cues of potassium homeostasis for stress tolerance and plant development, Biotechnology and Genetic Engineering Reviews, 40(4): 3527-3570.
Anwar S., Ashraf M., Saleem M., Shafiq F., Khan N., Khan R.A., Farid G., and Ashraf M., 2022, Integrated hormonal and nutrient management promote fruit retention and quality traits of Citrus reticulata, Journal of Plant Nutrition, 46(1): 83-100.
https://doi.org/10.1080/01904167.2022.2064301
Awad A.A., Hussein H.A., El Samad A.G.A., Belal H.E., and Beheiry H.R., 2024, Foliar nourishment with different potassium sources to maximize yield through improving nutrient uptake in Citrus aurantifolia trees grown in potassium-deficient soil, Journal of Soil Science and Plant Nutrition, 24(4): 7151-7166.
https://doi.org/10.1007/s42729-024-02030-2
Brital R., Ibriz M., Benmrich A.M., Benyahia H., Aboutayeb R., and Abail Z., 2024, Soil and leaf nutrient status of selected Valencia orange orchards in the Gharb Plain of Morocco, Agronomy, 14(12): 3040.
https://doi.org/10.3390/agronomy14123040
Chen F., Zheng S., Cui N., Wang Z., Jiang S., Tan M., Li H., Zhao L., and Liu C., 2026, Optimizing deficit irrigation and fertilization at growth stages to improve citrus yield, fruit quality, and water-fertilizer productivity in semi-arid Southwest China, Agricultural Water Management, 327: 110278.
https://doi.org/10.1016/j.agwat.2026.110278
Costa L., Kunwar S., Ampatzidis Y., and Albrecht U., 2022, Determining leaf nutrient concentrations in citrus trees using UAV imagery and machine learning, Precision Agriculture, 23(3): 854-875.
https://doi.org/10.1007/s11119-021-09864-1
Dreyer I., Gomez-Porras J.L., and Riedelsberger J., 2017, The potassium battery: A mobile energy source for transport processes in plant vascular tissues, New Phytologist, 216(4): 1049-1053.
https://doi.org/10.1111/nph.14667
Han H., Chen X.L., Liu Y.Z., Zhou T., Alam S.M., and Khan M.A., 2024, Foliar spraying magnesium promotes soluble sugar accumulation by inducing the activities of sucrose biosynthesis and transport in citrus fruits, Scientia Horticulturae, 324: 112593.
https://doi.org/10.1016/j.scienta.2023.112593
Hasanuzzaman M., Bhuyan M., Nahar K., Hossain M., Mahmud J., Hossen M.S., Masud A.A.C., Moumita M., and Fujita M., 2018, Potassium: A vital regulator of plant responses and tolerance to abiotic stresses, Agronomy, 8(3): 31.
https://doi.org/10.3390/agronomy8030031
Jiao Y., Sha C., and Shu Q., 2022, Integrated physiological and metabolomic analyses of the effect of potassium fertilizer on Citrus fruit splitting, Plants, 11(4): 499.
https://doi.org/10.3390/plants11040499
Jiao Y., Zhang S., Jin H., Wang Y., Jia Y., Zhang H., Jiang Y., Liao W., Chen L.S., and Guo J., 2023, Fruit quality assessment based on mineral elements and juice properties in nine citrus cultivars, Frontiers in Plant Science, 14: 1280495.
https://doi.org/10.3389/fpls.2023.1280495
Johnson R., Vishwakarma K., Hossen M.S., Kumar V., Shackira A., Puthur J.T., Abdi G., Sarraf M., and Hasanuzzaman M., 2022, Potassium in plants: Growth regulation, signaling, and environmental stress tolerance, Plant Physiology and Biochemistry, 172: 56-69.
https://doi.org/10.1016/j.plaphy.2022.01.001
Khan M.N., and Nabi G., 2023, Potassium fertilizer source and timing regulate growth, flowering and yield in trees of sweet lime (Citrus limetta L.), Sarhad Journal of Agriculture, 39(3): 655-664.
https://doi.org/10.17582/journal.sja/2023/39.3.655.664
Khan M.N., Nabi G., Khattak A., Ismail E.A.A., Awwad F.A., Irshad M., Ahmad H., and Suhail M., 2025, Efficacy of foliar application of potassium nitrate in the regulation of photosynthetic pigments, sex expression, yield and quality attributes of sweet lime (Citrus limmetoids), International Journal of Fruit Science, 25(1): 40-51.
https://doi.org/10.1080/15538362.2025.2519138
Kumar A.S., Kaniganti S., Kumari H.P., Reddy S.P., Suravajhala P., P S., and Kishor P.B.K., 2022, Functional and biotechnological cues of potassium homeostasis for stress tolerance and plant development, Biotechnology and Genetic Engineering Reviews, 40: 3527-3570.
https://doi.org/10.1080/02648725.2022.2143317
Kuzin A., and Solovchenko A., 2021, Essential role of potassium in apple and its implications for management of orchard fertilization, Plants, 10(12): 2624.
https://doi.org/10.3390/plants10122624
Kuzin A.I., Kashirskaya N.Y., Kochkina A.M., and Kushner A.V., 2020, Correction of potassium fertigation rate of apple tree (Malus domestica Borkh.) in Central Russia during the growing season, Plants, 9(10): 1366.
https://doi.org/10.3390/plants9101366
Lado J., Gambetta G., and Zacarias L., 2018, Key determinants of citrus fruit quality: Metabolites and main changes during maturation, Scientia Horticulturae, 233: 238-248.
https://doi.org/10.1016/j.scienta.2018.01.055
Li Z., Duan S., Xin O., Song S., Chen D., Fan X., Ding H., and Shen H., 2024, Coupled soil moisture management and alginate oligosaccharide strategies enhance citrus orchard production, water and potassium use efficiency by improving the rhizosphere soil environment, Agricultural Water Management, 297: 108828.
https://doi.org/10.1016/j.agwat.2024.108828
Lima Neto A.J.D., Krug A.V., Moura-Bueno J.M., Rozane D.E., Natale W., Hindersmann J., Marques A.L.L., Stefanello L., Papalia D., and Brunetto G., 2025, Proposal of critical nutrient levels in soil and citrus leaves using the boundary line method, Plants, 14(12): 1764.
https://doi.org/10.3390/plants14121764
Lu W., Hao W., Liu K., Liu J., Yin C., Su Y., Hang Z., Peng B., Liu H., Xiong B., Liao L., He J., Zhang M., Wang X., and Wang Z., 2024, Analysis of sugar components and identification of SPS genes in citrus fruit development, Frontiers in Plant Science, 15: 1372809.
https://doi.org/10.3389/fpls.2024.1372809
Luo A., Zhou C., and Chen J., 2021, The associated with carbon conversion rate and source–sink enzyme activity in tomato fruit subjected to water stress and potassium application, Frontiers in Plant Science, 12: 681145.
https://doi.org/10.3389/fpls.2021.681145
Ma X.C., Li F.F., Chen Y.W., Chang Y.Y., Lian X.F., Li Y.S., Ye L., Yin T., and Lu X.P., 2022, Effects of fertilization approaches on plant development and fertilizer use of citrus, Plants, 11(19): 2547.
https://doi.org/10.3390/plants11192547
Magbalot-Fernandez A., and De Guzman C., 2019, Phenology of ‘Magallanes’ pummelo (Citrus maxima) trees and its growth and development as influenced by potassium nutrition, Asian Journal of Research in Agriculture and Forestry, 3(4): 1-18.
https://doi.org/10.9734/ajraf/2019/v3i430043
Manzi M., Wlasiuk B., Pintos P., and Lado J., 2026, Potassium availability modulates magnesium and calcium accumulation during ‘Salustiana’ (Citrus sinensis) orange fruit development, Journal of Plant Nutrition: 1-15.
https://doi.org/10.1080/01904167.2026.2614511
Mao Z., Wang Y., Li M., Zhang S., Zhao Z., Xu Q., Liu J., and Li C., 2024, Vacuolar proteomic analysis reveals tonoplast transporters for accumulation of citric acid and sugar in citrus fruit, Horticulture Research, 11(1): uhad249.
https://doi.org/10.1093/hr/uhad249
Morales Alfaro J., Bermejo A., Navarro P., Quinones A., and Salvador A., 2023, Effect of rootstock on citrus fruit quality: A review, Food Reviews International, 39(5): 2835-2853.
https://doi.org/10.1080/87559129.2021.1978093
Nguyen H.H., and Tai T.N., 2020, Effects of combination between nitrogen and potassium fertilization on yield and quality of Valencia orange fruits, Journal of Agricultural Science, 12: 2019.
https://doi.org/10.5539/jas.v12n1p38
Papadakis I.E., Ladikou E.V., Oikonomou A., Chatzistathis T., and Chatziperou G., 2023, Exploring the impact of potassium on growth, photosynthetic performance, and nutritional status of lemon trees (cv. Adamopoulou) grafted onto sour orange and volkamer lemon rootstocks, Sustainability, 15(22): 15858.
https://doi.org/10.3390/su152215858
Quaggio J.A., Souza T.R., Zambrosi F.C., Mattos Jr D., Boaretto R.M., and Silva G., 2019, Citrus fruit yield response to nitrogen and potassium fertilization depends on nutrient-water management system, Scientia Horticulturae, 249: 329-333.
https://doi.org/10.1016/j.scienta.2019.02.001
Raddatz N., Morales de los Ríos L., Lindahl M., Quintero F.J., and Pardo J.M., 2020, Coordinated transport of nitrate, potassium, and sodium, Frontiers in Plant Science, 11: 247.
https://doi.org/10.3389/fpls.2020.00247
Sardans J., and Peñuelas J., 2021, Potassium control of plant functions: Ecological and agricultural implications, Plants, 10(2): 419.
https://doi.org/10.3390/plants10020419
Shah I.H., Manzoor M.A., Azam M., Wu J., Li X., Rehman A., Li P., Zhang Y., Niu Q., and Chang L., 2025, Comprehensive characterization and expression profiling of sucrose phosphate synthase (SPS) and sucrose synthase (SUS) family in Cucumis melo under the application of nitrogen and potassium, BMC Plant Biology, 25(1): 285.
https://doi.org/10.1186/s12870-025-06308-0
Shah I.H., Wu J., Li X., Hameed M., Manzoor M.A., Li P., Zhang Y., Niu Q., and Chang L., 2024, Exploring the role of nitrogen and potassium in photosynthesis implications for sugar: Accumulation and translocation in horticultural crops, Scientia Horticulturae, 327: 112832.
https://doi.org/10.1016/j.scienta.2023.112832
Shi X., Wen M., Dong Z., Zhang J., Srivastava A.K., Moussa M.G., and Zhang Y., 2025, Periodicity of fruit cracking in orange fruit and integrated management intervention, Plants, 14(3): 389.
https://doi.org/10.3390/plants14030389
Shrestha S., Waldo L., and Schumann A., 2025, Foliar spray of macronutrient influences fruit quality of Sugar Belle® mandarin grown in Florida sandy soil, Agronomy, 15(6): 1483.
https://doi.org/10.3390/agronomy15061483
Singh G., Rattanpal H.S., Chahal T.S., Singh K., and Gupta M., 2023, Effects of potassium application on vegetative growth, fruiting, and nutrient status of Kinnow mandarin under Indian sub-tropical conditions, Journal of Plant Nutrition, 46(7): 1197-1206.
https://doi.org/10.1080/01904167.2022.2068427
Spreen T.H., Gao Z., Fernandes Jr W., and Zansler M.L., 2020, Global economics and marketing of citrus products, In: The Genus Citrus, pp. 471-493, Woodhead Publishing.
https://doi.org/10.1016/b978-0-12-812163-4.00023-1
Stagno F., Brambilla M., Roccuzzo G., and Assirelli A., 2024, Water use efficiency in a deficit-irrigated orange orchard, Horticulturae, 10(5): 498.
https://doi.org/10.3390/horticulturae10050498
Tahir M.M., Sabah N., Gul S., Javed M., Aslam M., Daud M.A., Aziz A., and Javed M., 2023, Optimization of new generation potassium (NG-K) fertilizer for improvement in quantity and quality of citrus (Citrus limon), SABRAO Journal of Breeding and Genetics, 55(2): 575-586.
https://doi.org/10.54910/sabrao2023.55.2.29
Thu A.M., Alam S.M., Khan M.A., Han H., Liu D., Tahir R., Ateeq M., and Liu Y.-Z., 2024, Foliar spraying of potassium sulfate during fruit development comprehensively improves the quality of citrus fruits, Scientia Horticulturae, 338: 113696.
https://doi.org/10.1016/j.scienta.2024.113696
Toor M.D., Gondal A.H., Javid M.S., Ashraf M.W., Hussain I., and Bakar A., 2021, Potassium as an essential nutrient for citrus plant: A review, Acta Scientific Agriculture, 5(7).
https://doi.org/10.31080/asag.2021.05.1024
Tränkner M., Tavakol E., and Jákli B., 2018, Functioning of potassium and magnesium in photosynthesis, photosynthate translocation and photoprotection, Physiologia Plantarum, 163(3): 414-431.
https://doi.org/10.1111/ppl.12747
Valizadehkaji B., and Mohammaei M., 2025, Foliar application of biostimulants and potassium silicate enhances yield and fruit quality of mandarin cv. ‘Page’, Applied Fruit Science, 67(1): 8.
https://doi.org/10.1007/s10341-024-01242-1
Venkateswara S.M., and Padmanaban J., 2025, Interpretable deep learning models for independent fertilizer and crop recommendation, Scientific Reports, 15(1): 41721.
https://doi.org/10.1038/s41598-025-26910-4
Wang J., Lu Y., Zhang X., Hu W., Lin L., Deng Q., Xia H., Liang D., and Lv X., 2024, Effects of potassium-containing fertilizers on sugar and organic acid metabolism in grape fruits, International Journal of Molecular Sciences, 25(5): 2828.
https://doi.org/10.3390/ijms25052828
Wang Y., Long Q., Li Y., Kang F., Fan Z., Xiong H., Zhao H., Luo Y., Guo R., He X., Lakshmanan P., Shi X., Zhang F., and Zhang Y., 2022, Mitigating magnesium deficiency for sustainable citrus production: A case study in Southwest China, Scientia Horticulturae, 295: 110832.
https://doi.org/10.1016/j.scienta.2021.110832
Wegner L.H., Pottosin I., Dreyer I., and Shabala S., 2025, Potassium homeostasis and signalling: From the whole plant to the subcellular level, Quantitative Plant Biology, 6: e13.
https://doi.org/10.1017/qpb.2025.10
Wen M., Zhang J., Zheng Y., and Yi S., 2021, Effects of combined potassium and organic fertilizer application on Newhall navel orange nutrient uptake, yield, and quality, Agronomy, 11(10): 1990.
https://doi.org/10.3390/agronomy11101990
Wu K., Hu C., Liao P., Hu Y., Sun X., Tan Q., Pan Z., Xu S., Dong Z., and Wu S., 2024, Potassium stimulates fruit sugar accumulation by increasing carbon flow in Citrus sinensis, Horticulture Research, 11(11): uhae240.
https://doi.org/10.1093/hr/uhae240
Wu K., Hu C., Wang J., Guo J., Sun X., Tan Q., Zhao X., and Wu S., 2023, Comparative effects of different potassium sources on soluble sugars and organic acids in tomato, Scientia Horticulturae, 308: 111601.
https://doi.org/10.1016/j.scienta.2022.111601
Wu S., Zhang C., Li M., Tan Q., Sun X., Pan Z., Deng X., and Hu C., 2021, Effects of potassium on fruit soluble sugar and citrate accumulations in Cara Cara navel orange (Citrus sinensis L. Osbeck), Scientia Horticulturae, 283: 110057.
https://doi.org/10.1016/j.scienta.2021.110057
Xu H., Wang Y., Luo Z., Hu W., Liao W., Chen L.-S., Li Y., and Guo J., 2024, Optimized nutrients management improved citrus yield and fruit quality in China: A meta-analysis, Ying Yong Sheng Tai Xue Bao (The Journal of Applied Ecology), 35(5): 1301-1311.
https://doi.org/10.13287/j.1001-9332.202405.011
Zayani A., Laasli S.E., Lahlali R., El Bouchtaoui F., and El Alem N., 2024, Contribution to the optimization of citrus (Citrus clementina Hort. Ex Tanaka) fruit fertilization using mobile lysimetry in orchards of the Souss-Massa region, Morocco, Journal of Applied and Natural Science, 16(1): 172.
https://doi.org/10.31018/jans.v16i1.5307
Zhang W., Zhang X., Wang Y., Zhang N., Guo Y., Ren X., and Zhao Z., 2018, Potassium fertilization arrests malate accumulation and alters soluble sugar metabolism in apple fruit, Biology Open, 7(12): bio024745.
https://doi.org/10.1242/bio.024745
Öz U., 2024, Genomic exploration of HAK/KUP/KT potassium transporter genes in Citrus sinensis (L.) Osbeck: A comprehensive bioinformatics approach, Journal of New Results in Science, 13(3): 186-200.
https://doi.org/10.54187/jnrs.1553782
Ülker T., and Kamiloğlu M.U., 2021, Influences of girdling and potassium treatments on fruit quality and some physiological characters of ‘Fremont’ mandarin variety, Folia Horticulturae, 33(1): 195-202.
https://doi.org/10.2478/fhort-2021-0015


. PDF(945KB)
. FPDF(win)
. FPDF(mac)
. HTML
. Online fPDF
Associated material
. Readers' comments
Other articles by authors
. Bo Zhang

Related articles
. Citrus
. Potassium management
. Fruit quality
. Sugar accumulation
. Precision fertilization
Tools
. Email to a friend
. Post a comment